Share
Convergent glycerolipid metabolism in highland adapted maize?
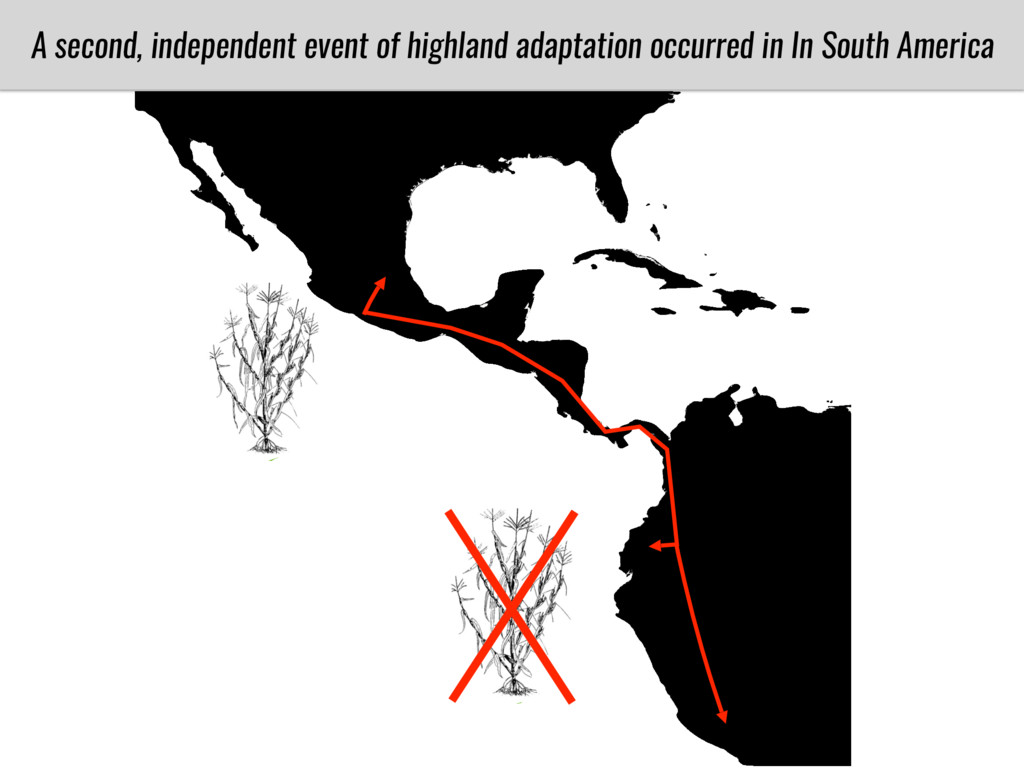
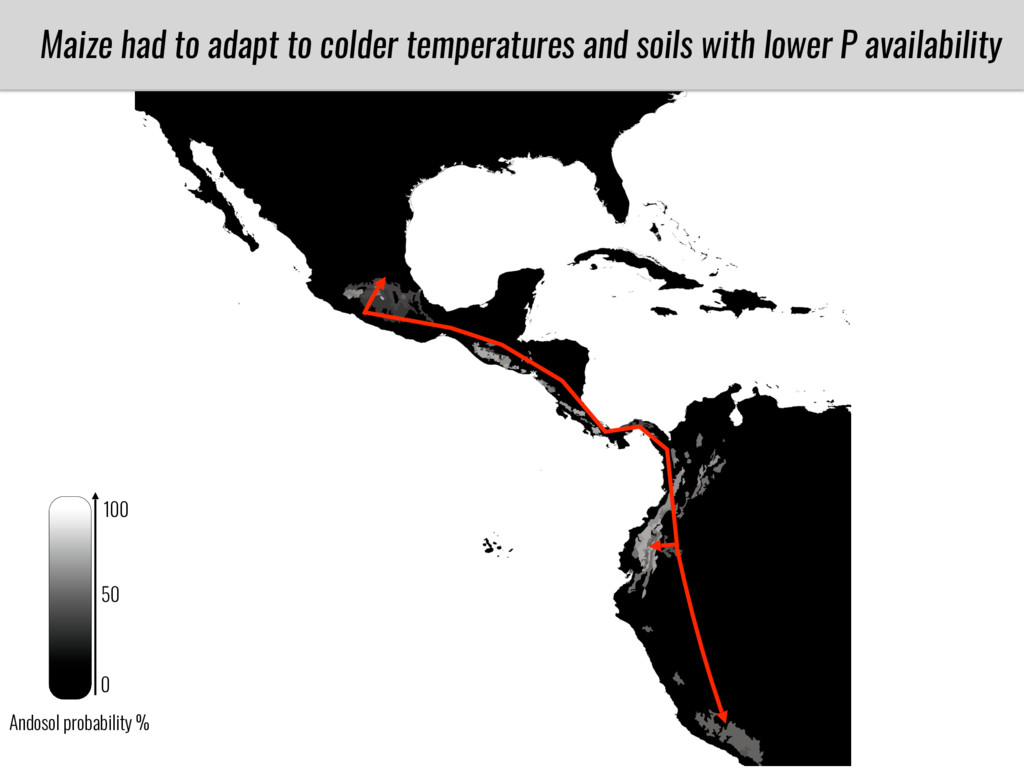
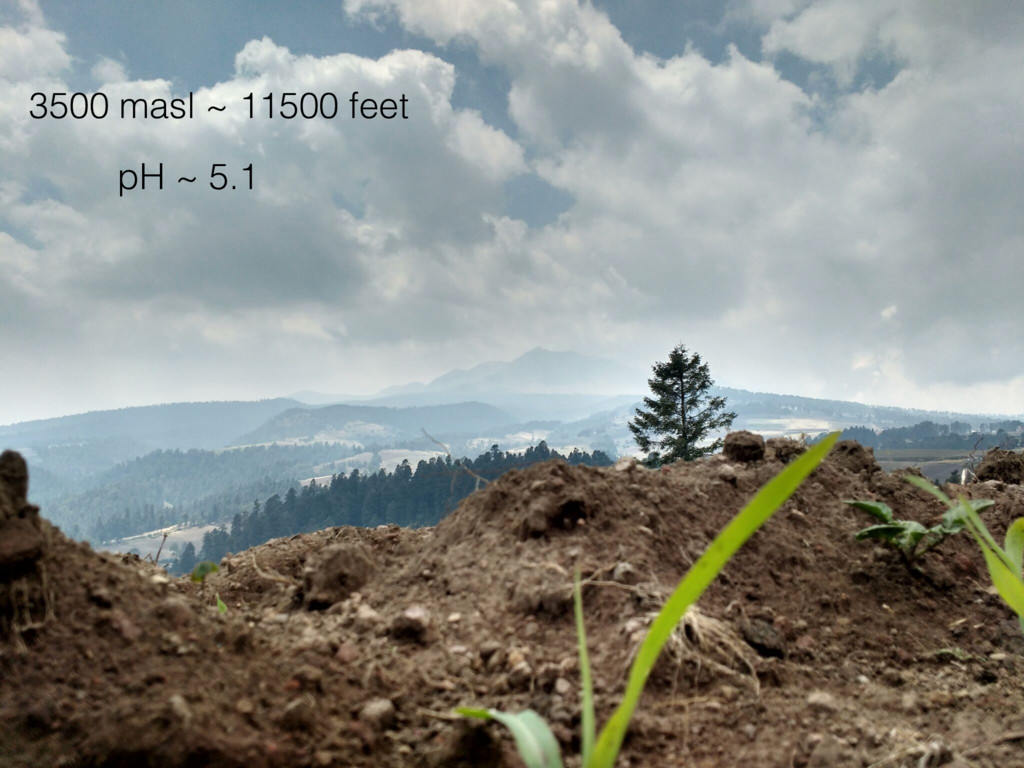
After domestication from lowland teosinte in Mexican subtropic maize colonized the highlands of both Mexico and South America characterized by lower temperatures and phosphorus bioavailability. We hypothesize that low temperature and phosphorus bioavailability were major selective forces during maize adaptation to the highlands and shaped glycerolipid metabolism since low temperature and P deficiency have opposite effects on the content of glycerolipid species.
To test this hypothesis grew a maize RIL mapping population (developed using a Mexican highland landrace Palomero Toluqueño and B73) and a 120 landrace diversity panel (composed of lowland and highland Mesoamerican and South American landraces) in common garden experiments at sea level and at 2600 masl. in Mexico and measures glycerolipid species (125 different compounds) that were used as phenotypes to identify genotype-phenotype associations and plasticity between highland and lowland conditions. I will present this results and in particular on an interesting QTL in ch3 that explains phosphatidylcholine to lysophosphatidylcholine conversion and seems to be selected against in highland Mexican landraces but not in South American ones.
Rubén Rellán Álvarez
Transcript
91 slides
-
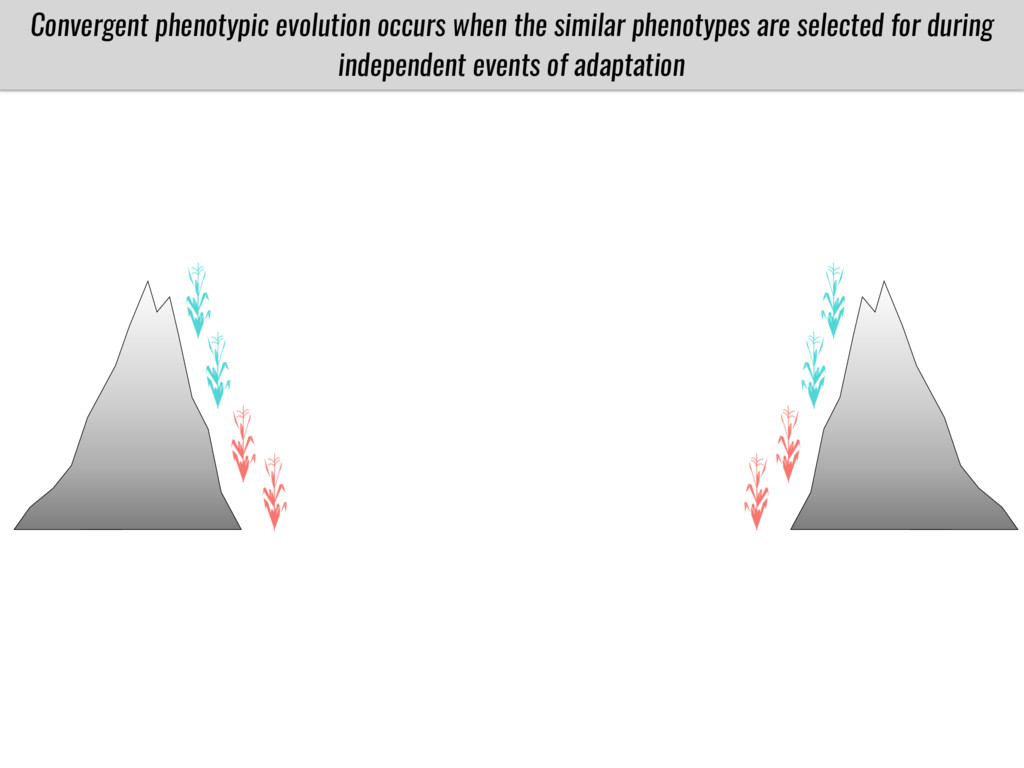
Convergent phenotypic evolution occurs when the similar phenotypes are selected
for during independent events of adaptation -
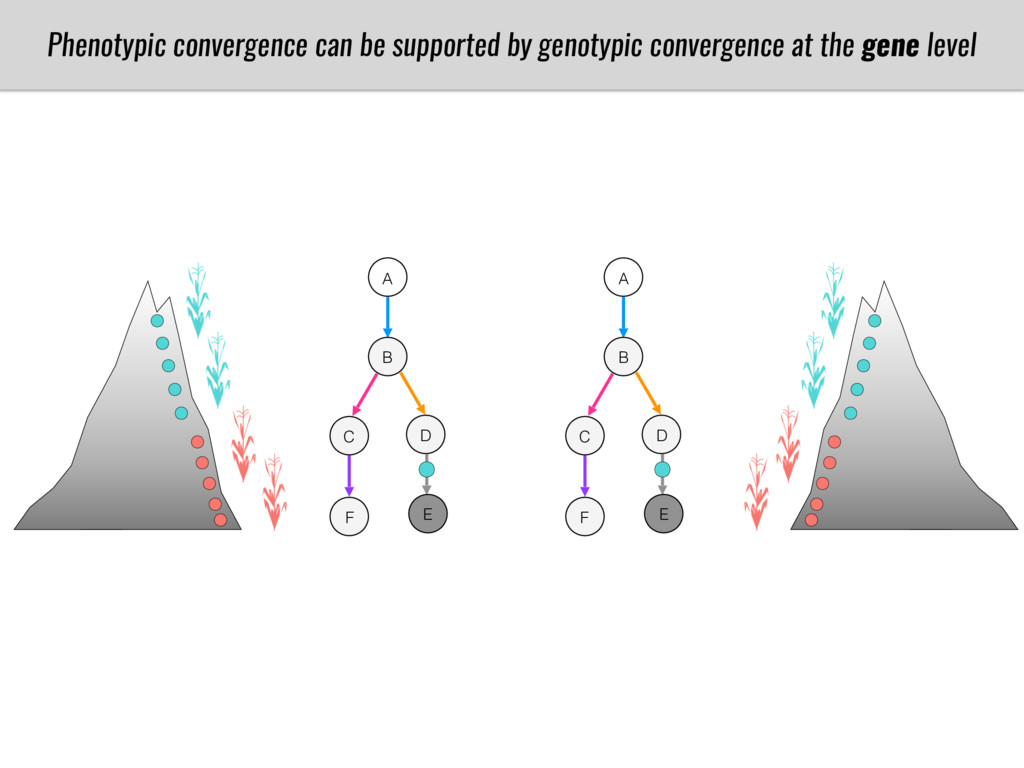
A B C D E F Phenotypic convergence can be
supported by genotypic convergence at the gene level A B C D E F -
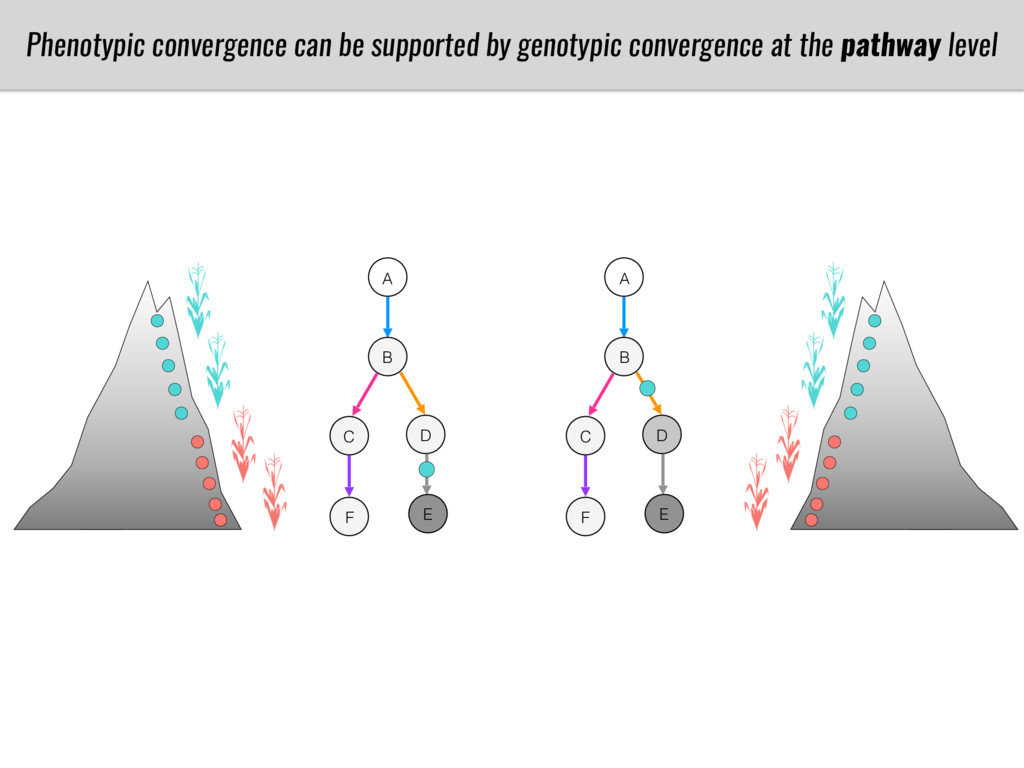
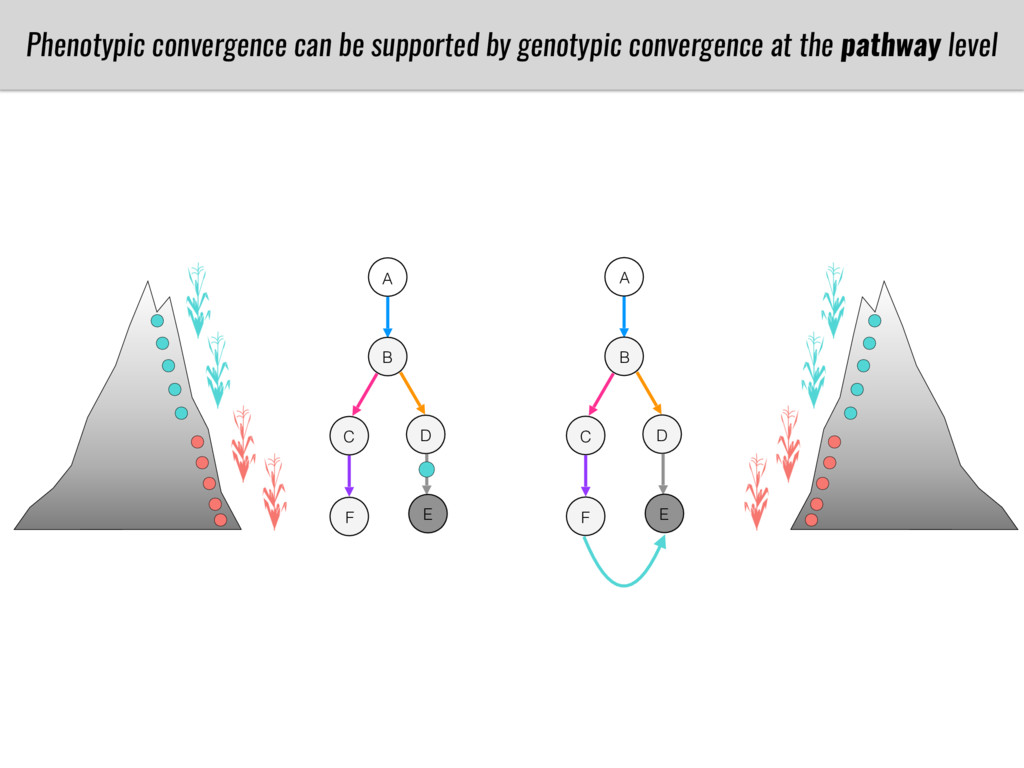
A B C D E F Phenotypic convergence can be
supported by genotypic convergence at the pathway level A B C D E F -
A B C D E F A B C D
E F Phenotypic convergence can be supported by genotypic convergence at the pathway level -
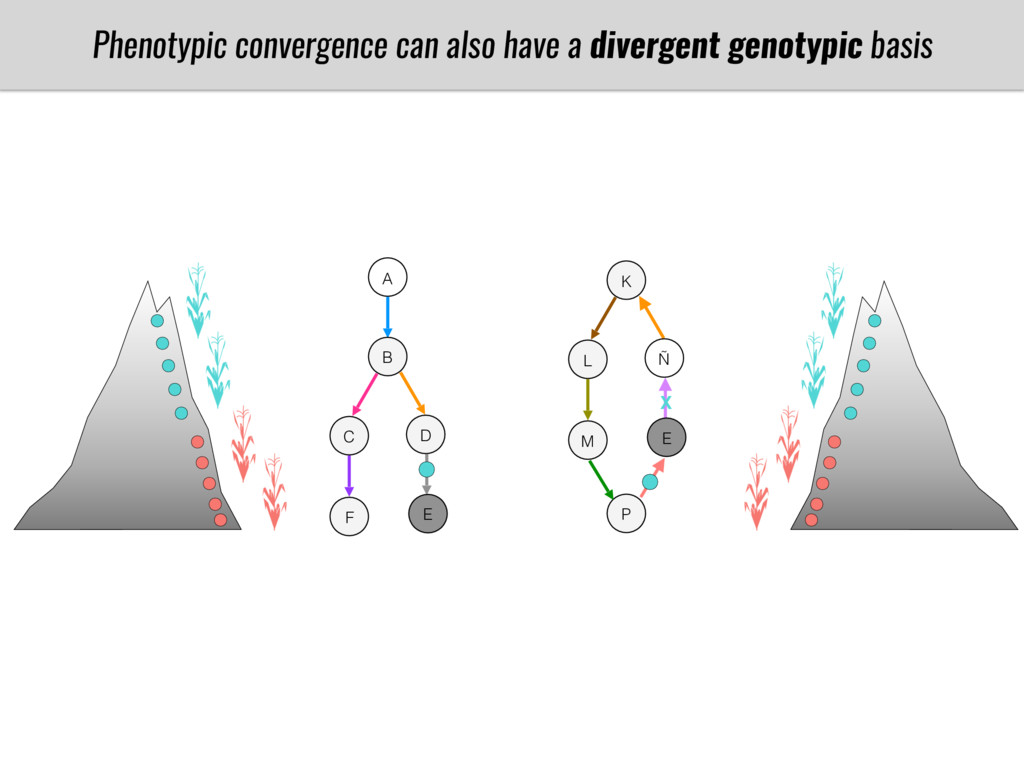
A B C D E F Phenotypic convergence can also
have a divergent genotypic basis K L Ñ E M P X -
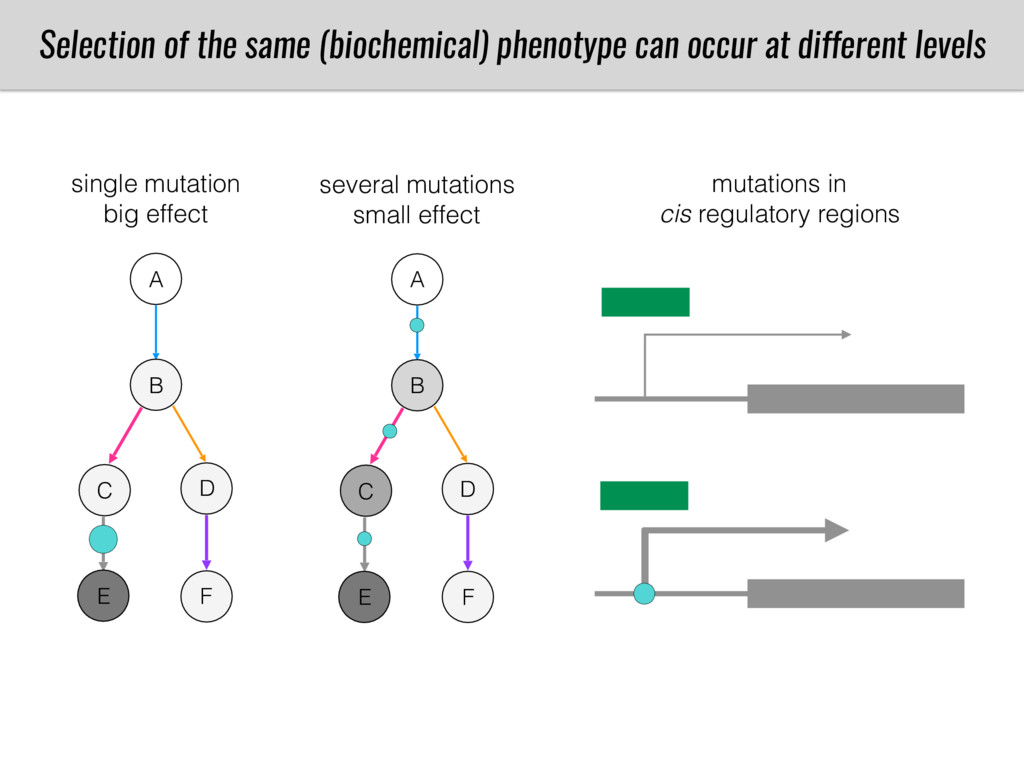
Selection of the same (biochemical) phenotype can occur at different
levels A B C D F A B C D E F single mutation big effect several mutations small effect mutations in cis regulatory regions E -
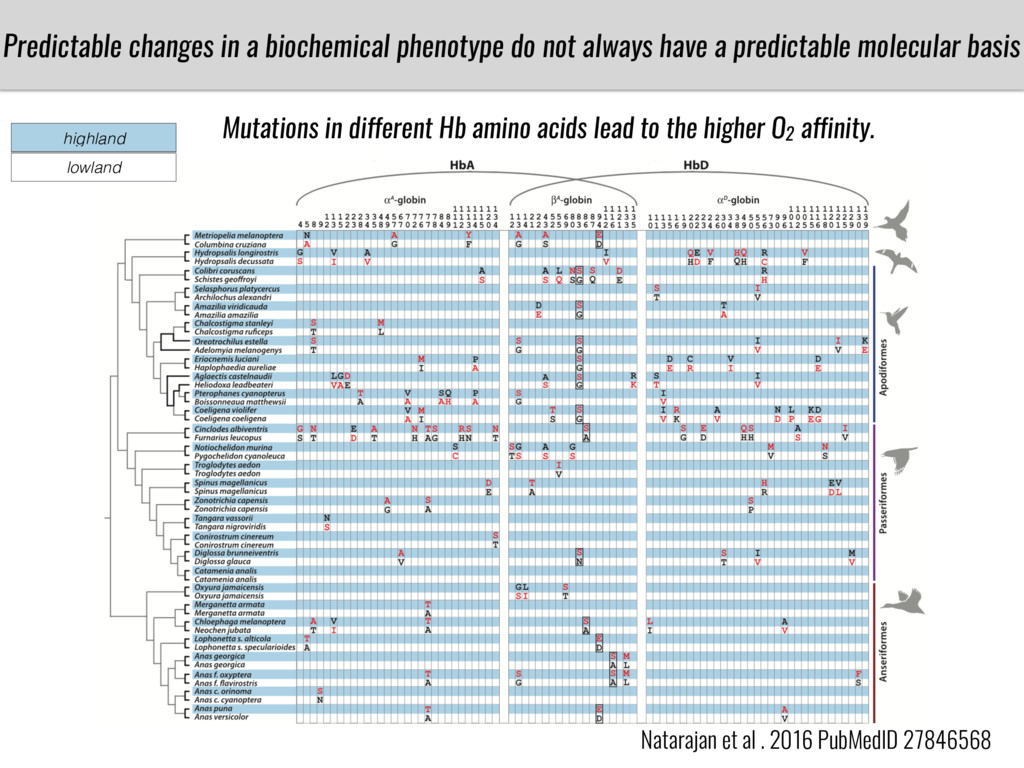
Predictable changes in a biochemical phenotype do not always have
a predictable molecular basis highland lowland Natarajan et al . 2016 PubMedID 27846568 Mutations in different Hb amino acids lead to the higher O2 affinity. -
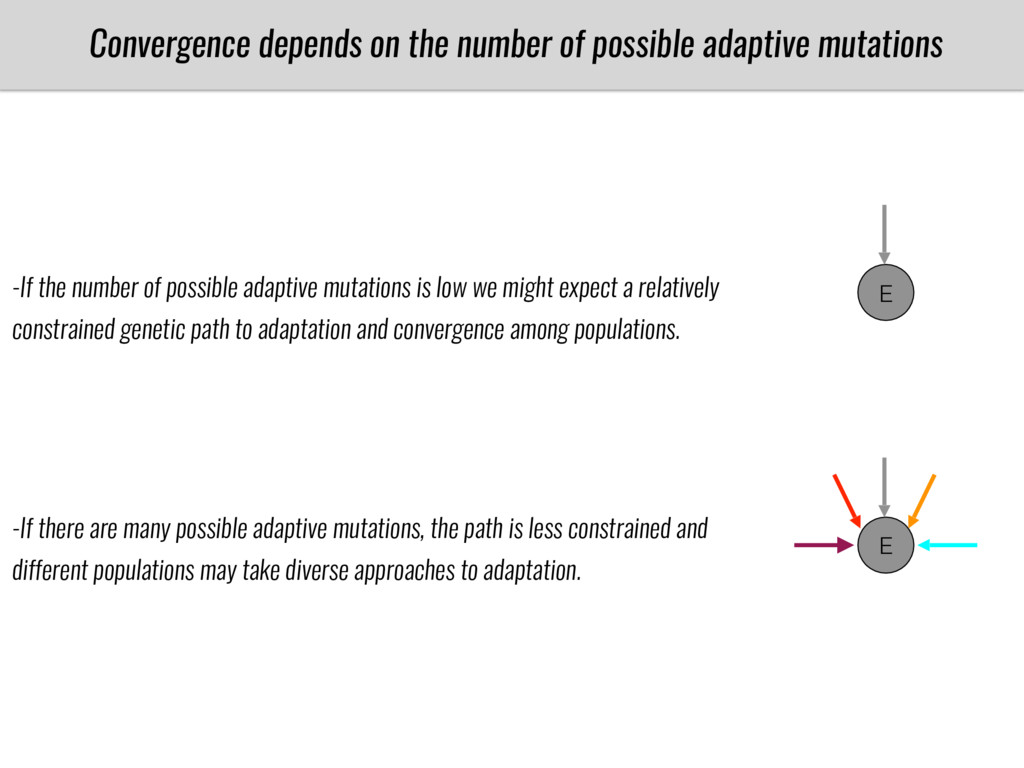
-If the number of possible adaptive mutations is low we
might expect a relatively constrained genetic path to adaptation and convergence among populations. -If there are many possible adaptive mutations, the path is less constrained and different populations may take diverse approaches to adaptation. Convergence depends on the number of possible adaptive mutations E E -
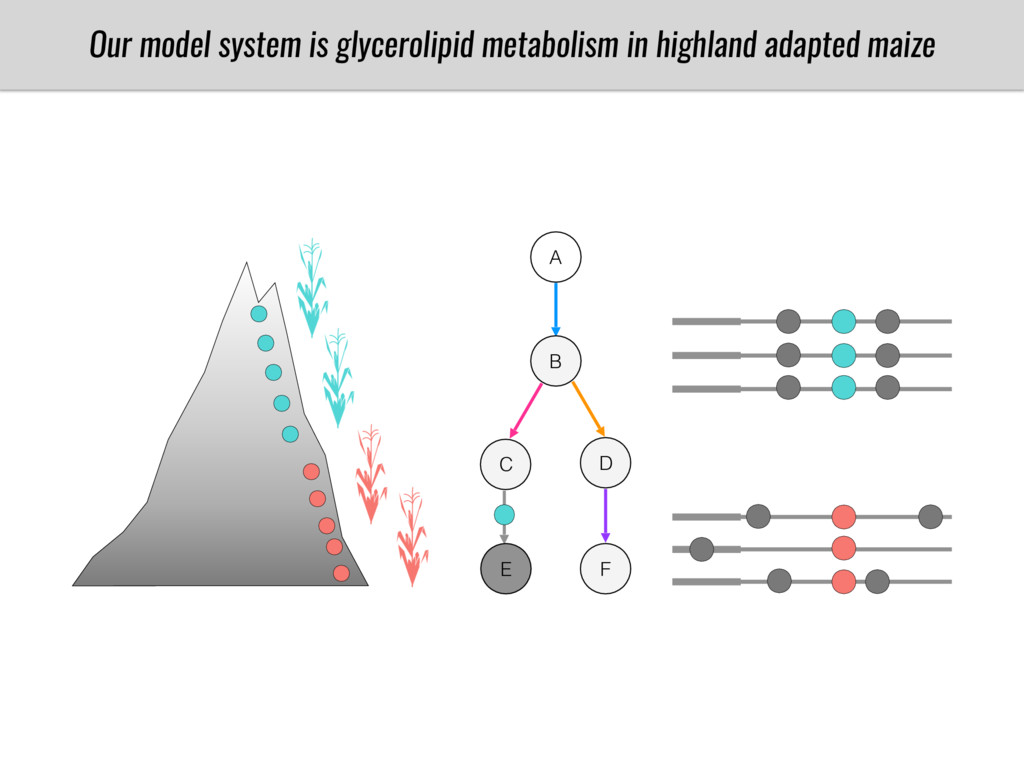
A B C D E F Our model system is
glycerolipid metabolism in highland adapted maize -
Maize colonized highland territory after its domestication in tropical areas
of Southwest Mexico Sawers et al . 2013 PubMedID 22303349 Relationships in the genus Zea Tripsicum Zea nicaraguensis Zea luxurians Zea diploperennis Zea perennis Zea mays ssp. huehuetenangensis Zea mays ssp. mexicana Zea mays ssp. parviglumis Zea mays ssp. mays After Hufford et al., 2012 -
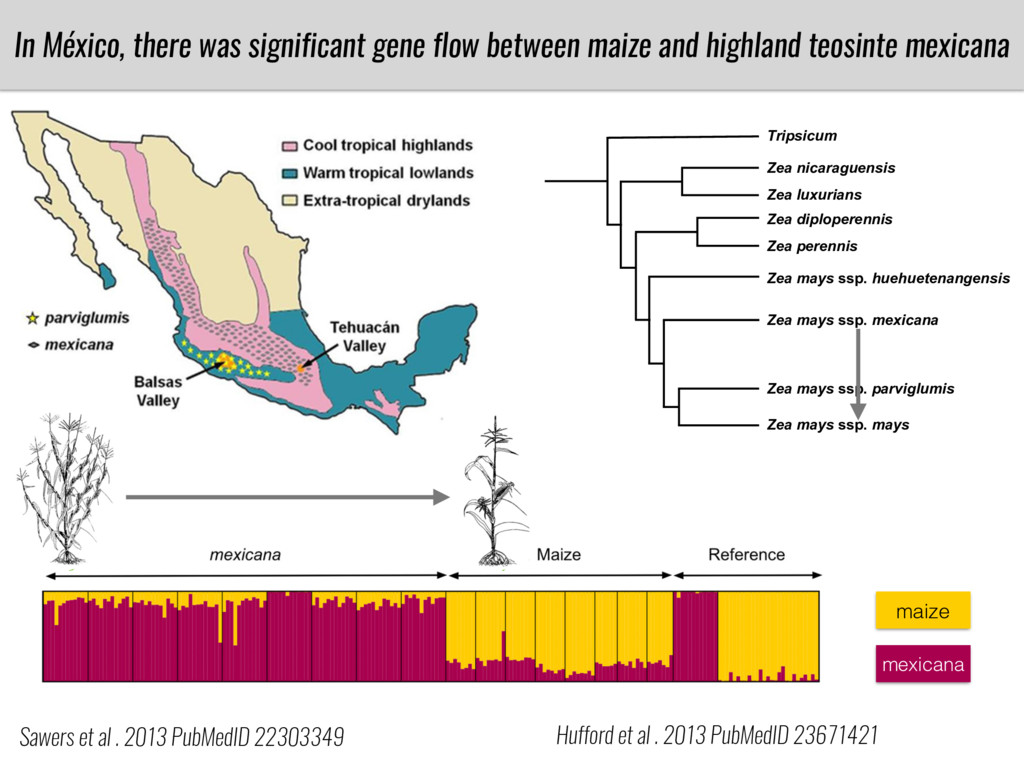
Relationships in the genus Zea Tripsicum Zea nicaraguensis Zea luxurians
Zea diploperennis Zea perennis Zea mays ssp. huehuetenangensis Zea mays ssp. mexicana Zea mays ssp. parviglumis Zea mays ssp. mays After Hufford et al., 2012 In México, there was significant gene flow between maize and highland teosinte mexicana Sawers et al . 2013 PubMedID 22303349 Hufford et al . 2013 PubMedID 23671421 maize mexicana low from mexicana in highland adaptation 3 parviglumis mexicana Geneflow from mexicana Adaptive? van Heerwaarden et al., 2011 Sawers & Sanchez, 2011 1750m parviglumis Gene flow from mexicana in highland adaptation 3 parviglumis mexicana Geneflow from mexicana Adaptive? van Heerwaarden et al., 2011 Sawers & Sanchez, 2011 1750m parviglumis -
3 parviglumis Geneflow from mexicana Adaptive? van Heerwaarden et al.,
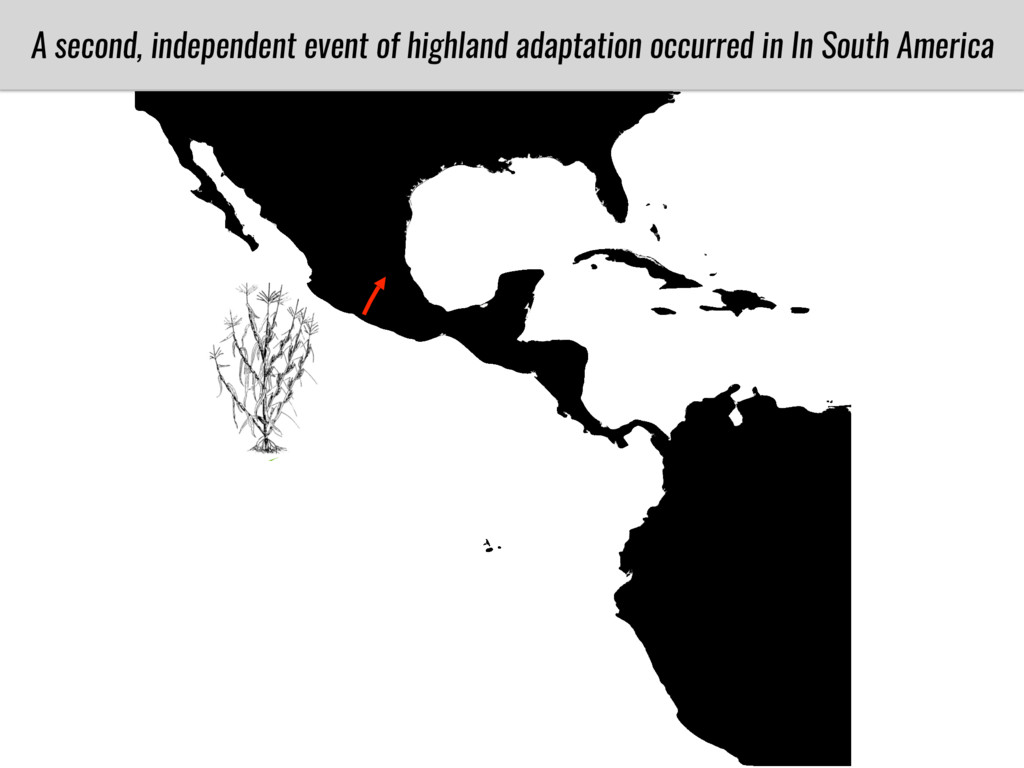
2011 Sawers & Sanchez, 2011 1750m parviglumis A second, independent event of highland adaptation occurred in In South America -
3 parviglumis Geneflow from mexicana Adaptive? van Heerwaarden et al.,
2011 Sawers & Sanchez, 2011 1750m parviglumis A second, independent event of highland adaptation occurred in In South America Gene flow from mexicana in highland a parviglumis Geneflow from mexicana Adaptive? van Heerwaarden et al., 2011 Sawers & Sanchez, 2011 parvig -
Andosol probability % 0 50 100 Maize had to adapt
to colder temperatures and soils with lower P availability -
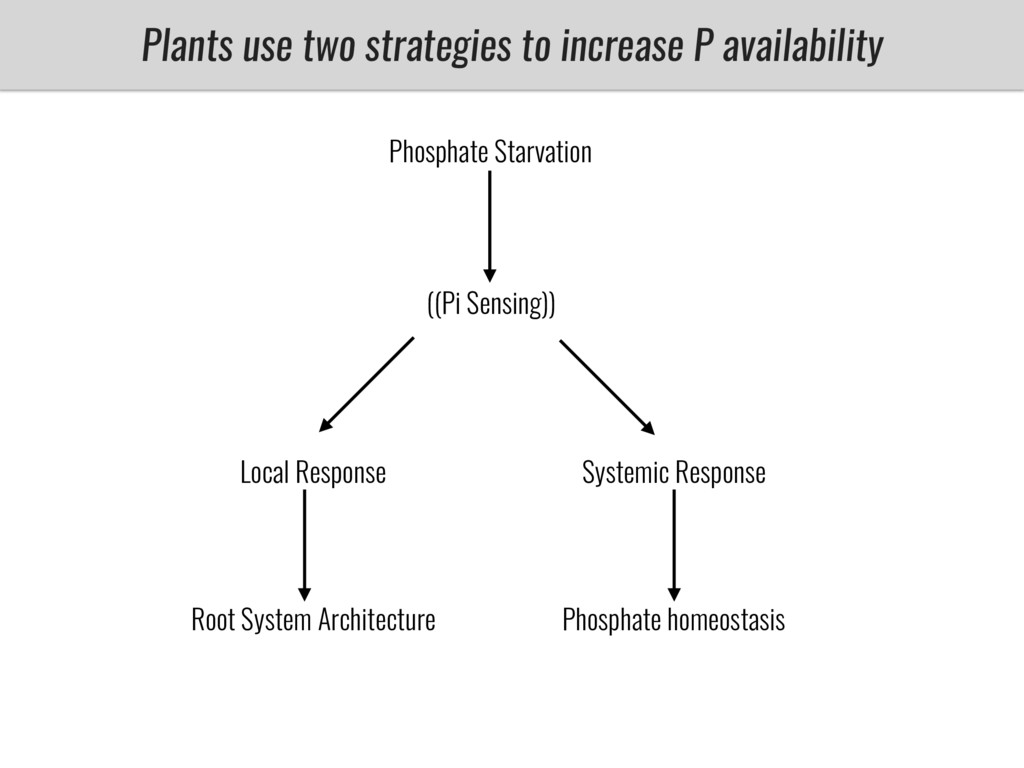
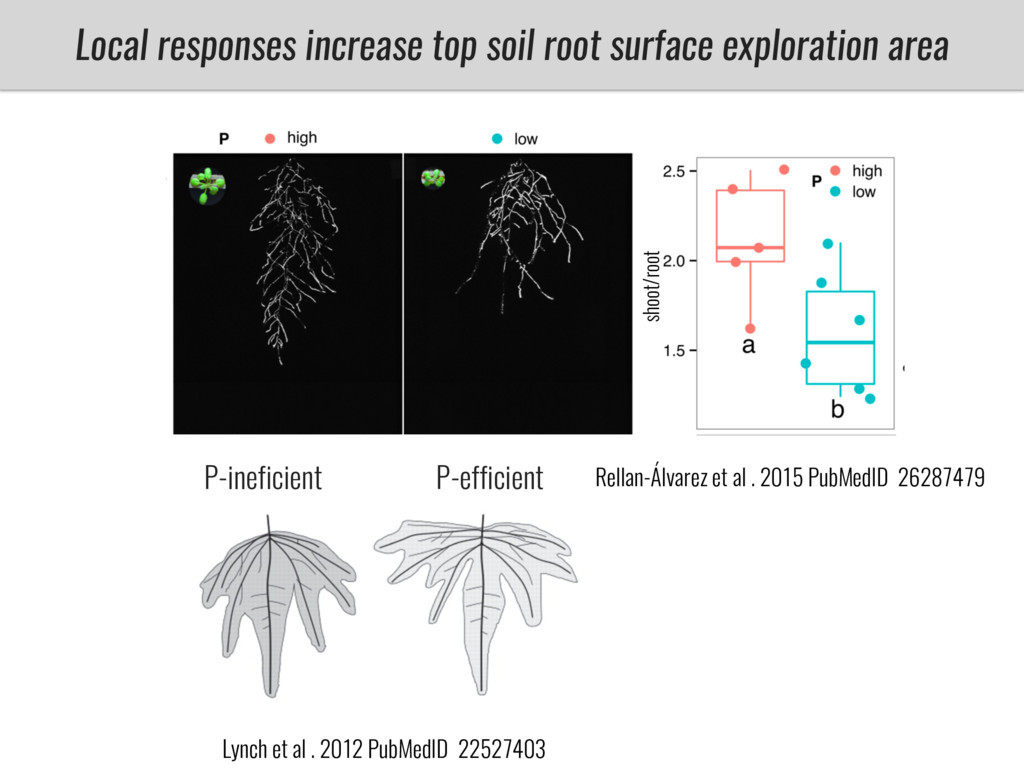
Plants use two strategies to increase P availability Phosphate Starvation
((Pi Sensing)) Local Response Systemic Response Root System Architecture Phosphate homeostasis -
Local responses increase top soil root surface exploration area P-ineficient
P-efficient Lynch et al . 2012 PubMedID 22527403 Rellan-Álvarez et al . 2015 PubMedID 26287479 shoot/root -
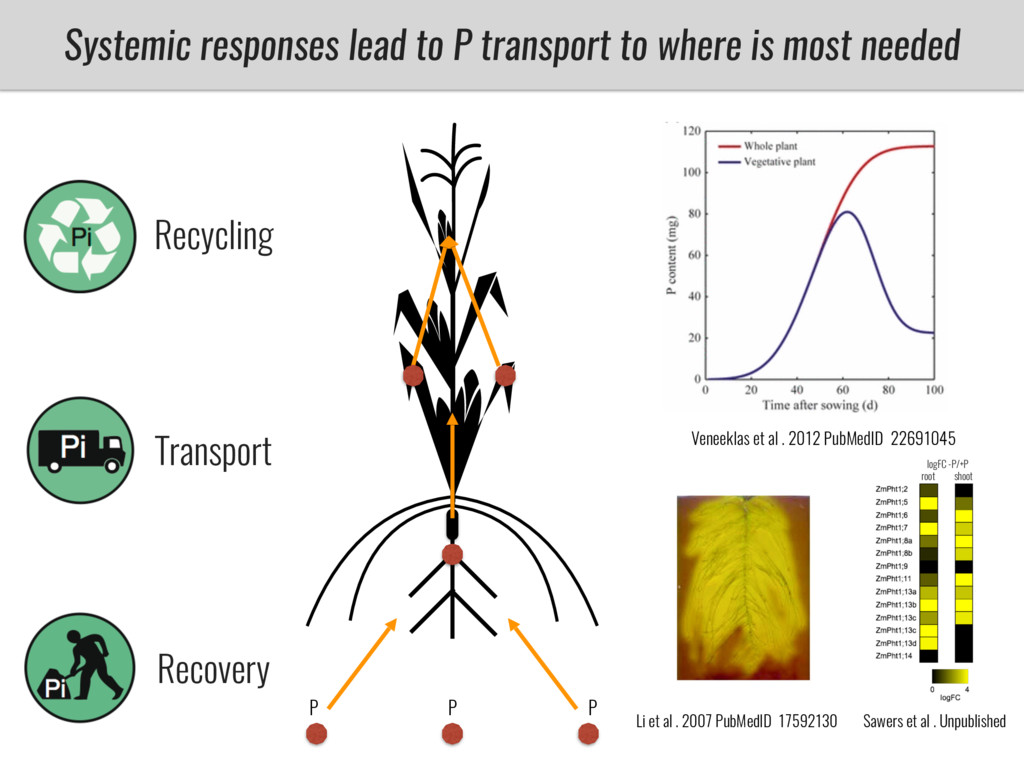
Recovery Transport Recycling Systemic responses lead to P transport to
where is most needed Li et al . 2007 PubMedID 17592130 logFC -P/+P root shoot Sawers et al . Unpublished Veneeklas et al . 2012 PubMedID 22691045 P P P -
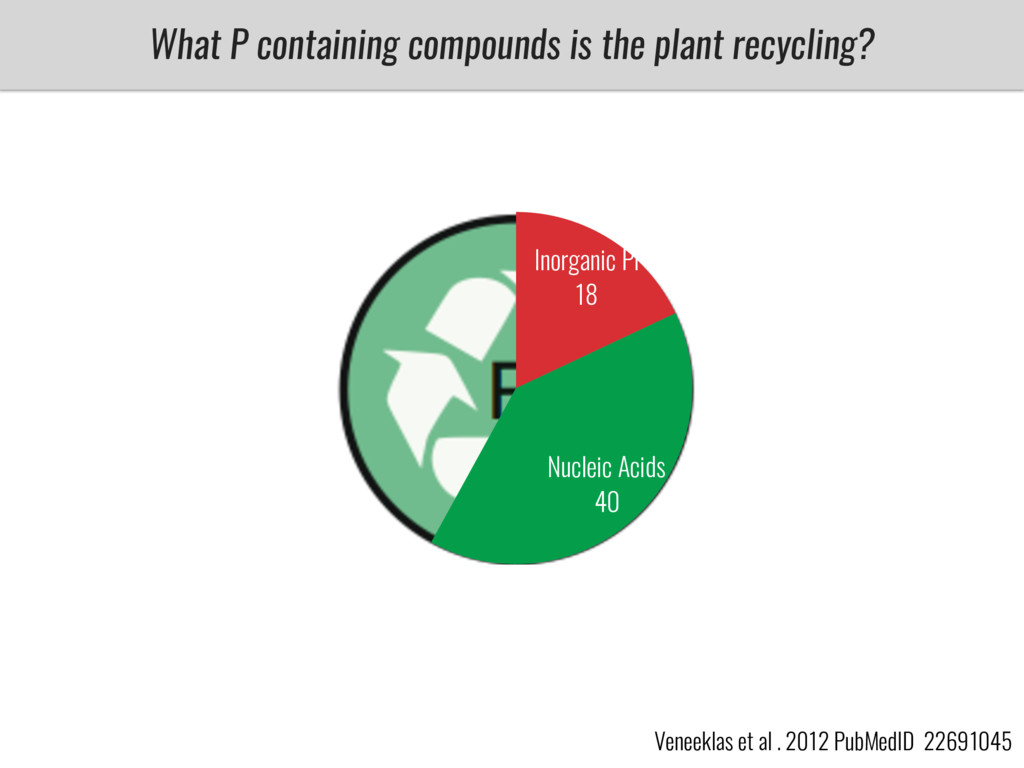
What P containing compounds is the plant recycling? Veneeklas et
al . 2012 PubMedID 22691045 -
What P containing compounds is the plant recycling? Veneeklas et
al . 2012 PubMedID 22691045 -
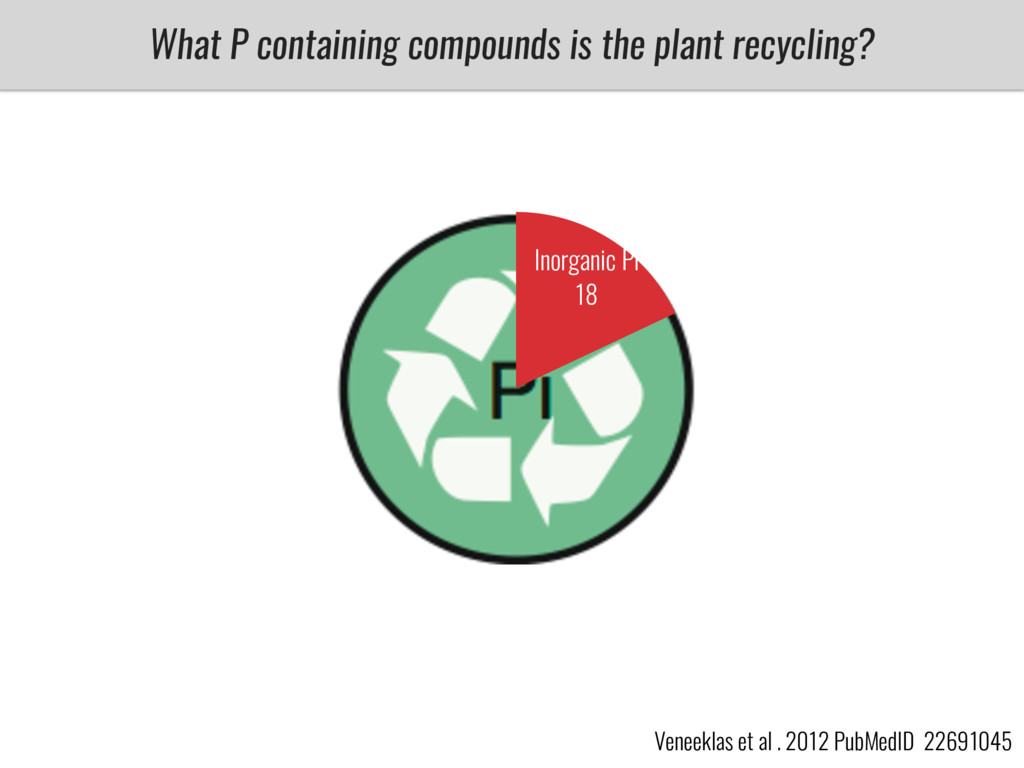
Inorganic Pi 18 What P containing compounds is the plant
recycling? Veneeklas et al . 2012 PubMedID 22691045 -
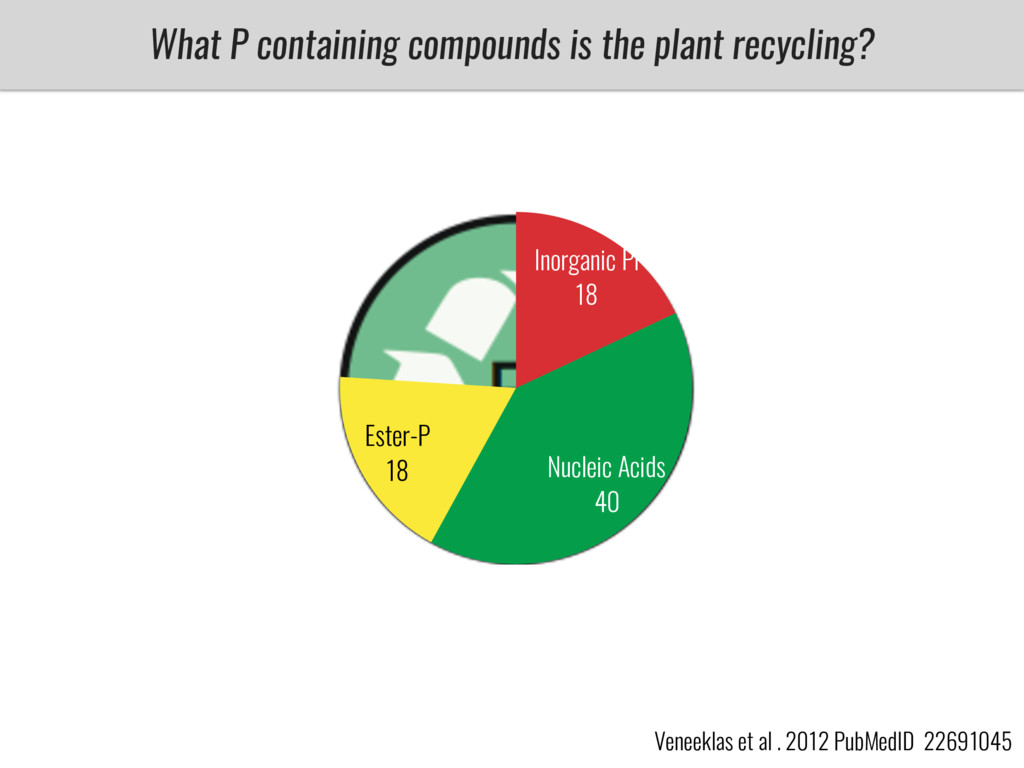
Nucleic Acids 40 Inorganic Pi 18 What P containing compounds
is the plant recycling? Veneeklas et al . 2012 PubMedID 22691045 -
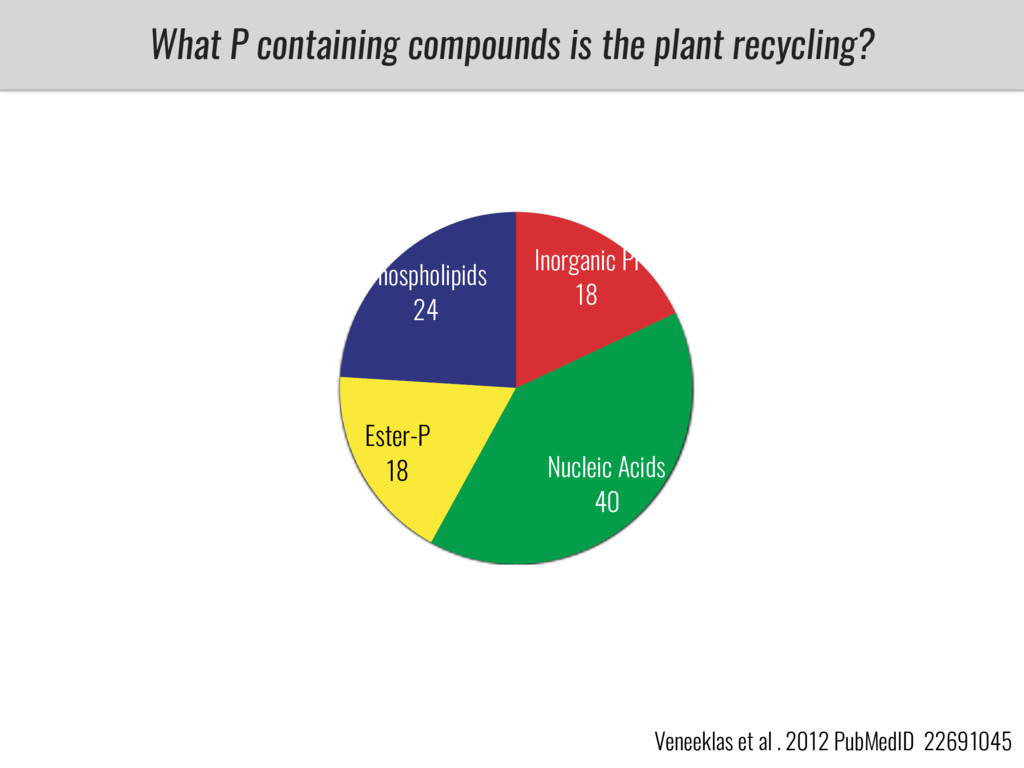
Ester-P 18 Nucleic Acids 40 Inorganic Pi 18 What P
containing compounds is the plant recycling? Veneeklas et al . 2012 PubMedID 22691045 -
Phospholipids 24 Ester-P 18 Nucleic Acids 40 Inorganic Pi 18
What P containing compounds is the plant recycling? Veneeklas et al . 2012 PubMedID 22691045 -
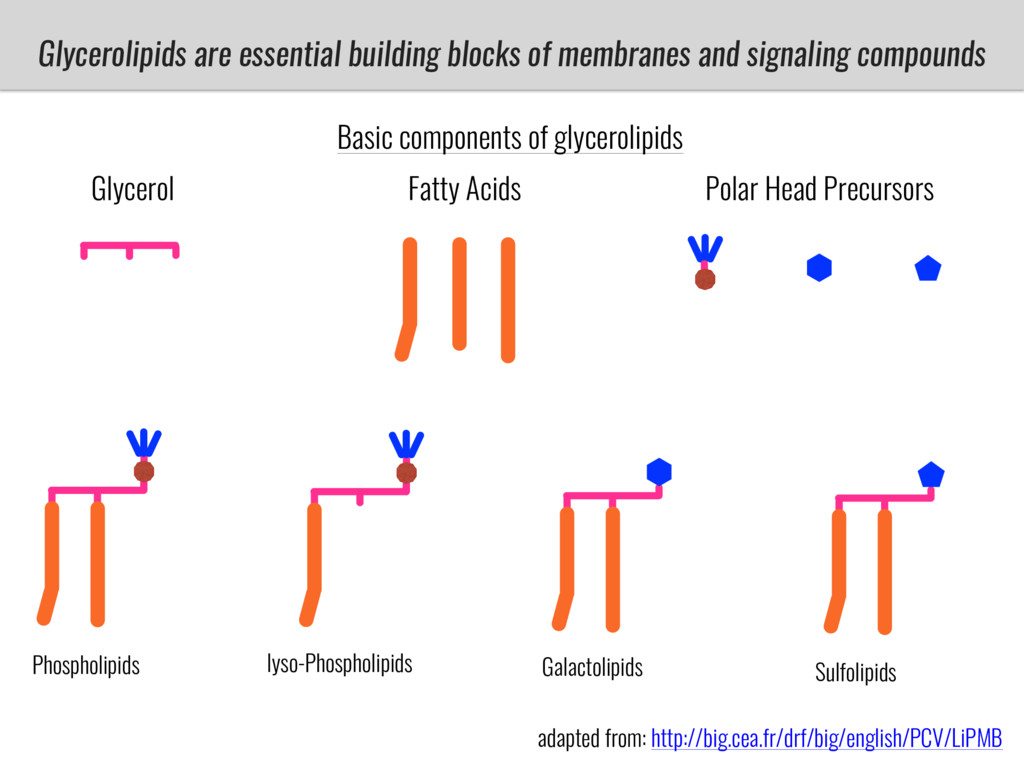
Glycerolipids are essential building blocks of membranes and signaling compounds
Glycerol Polar Head Precursors Fatty Acids Phospholipids Galactolipids Sulfolipids adapted from: http://big.cea.fr/drf/big/english/PCV/LiPMB Basic components of glycerolipids lyso-Phospholipids -
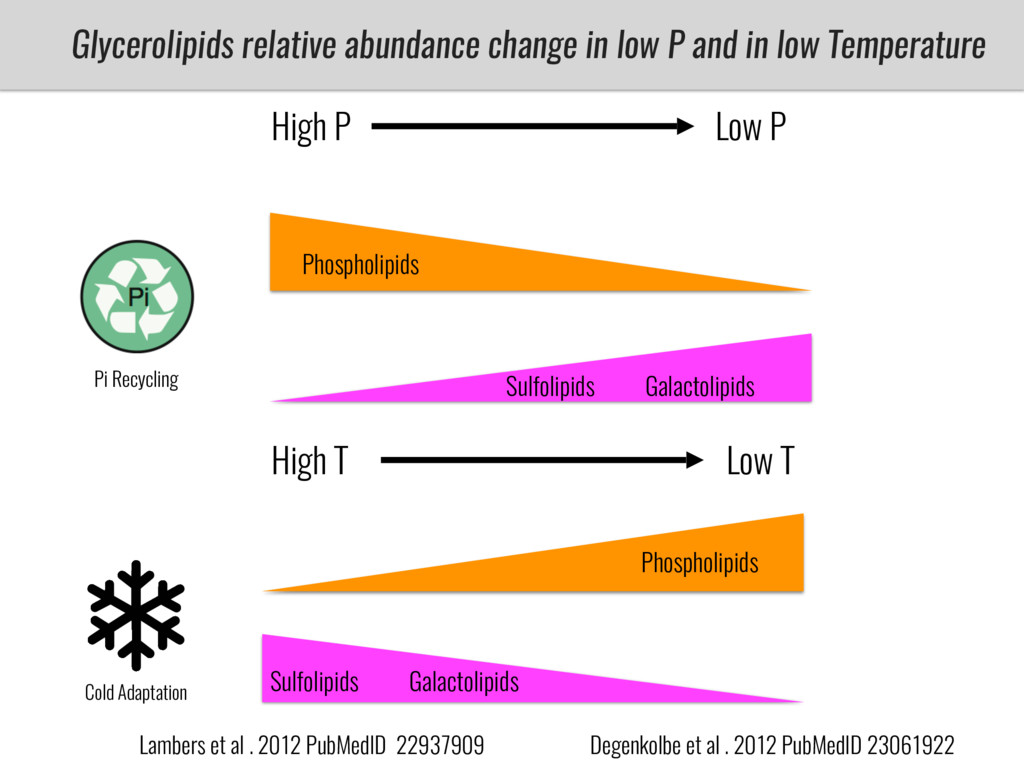
High P Low P Pi Recycling Cold Adaptation Glycerolipids relative
abundance change in low P and in low Temperature Lambers et al . 2012 PubMedID 22937909 Degenkolbe et al . 2012 PubMedID 23061922 Phospholipids Sulfolipids Galactolipids -
High P Low P Pi Recycling Cold Adaptation Glycerolipids relative
abundance change in low P and in low Temperature Lambers et al . 2012 PubMedID 22937909 Degenkolbe et al . 2012 PubMedID 23061922 Phospholipids Sulfolipids Galactolipids High T Low T Phospholipids Sulfolipids Galactolipids -
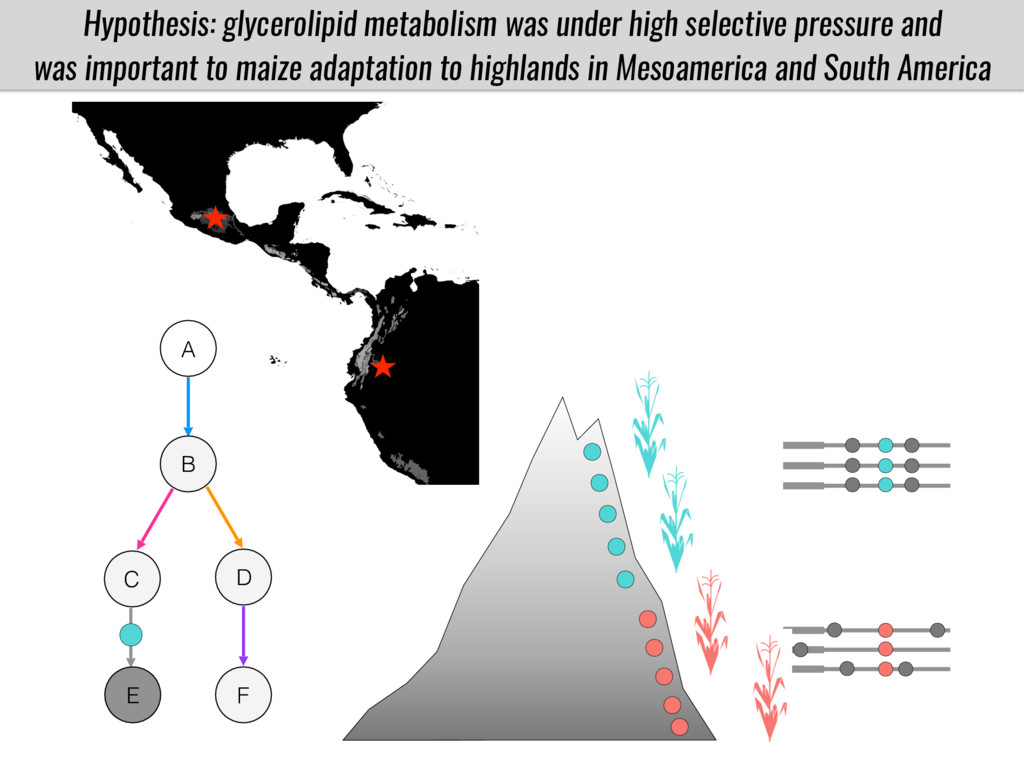
Hypothesis: glycerolipid metabolism was under high selective pressure and was
important to maize adaptation to highlands in Mesoamerica and South America A B C D E F -
Experimental approaches Common Garden Experiments in contrasting environments Bi-parental and
diversity panel mapping populations Biochemical phenotyping Quantitative and population genetics Reverse genetics and heterologous expression -
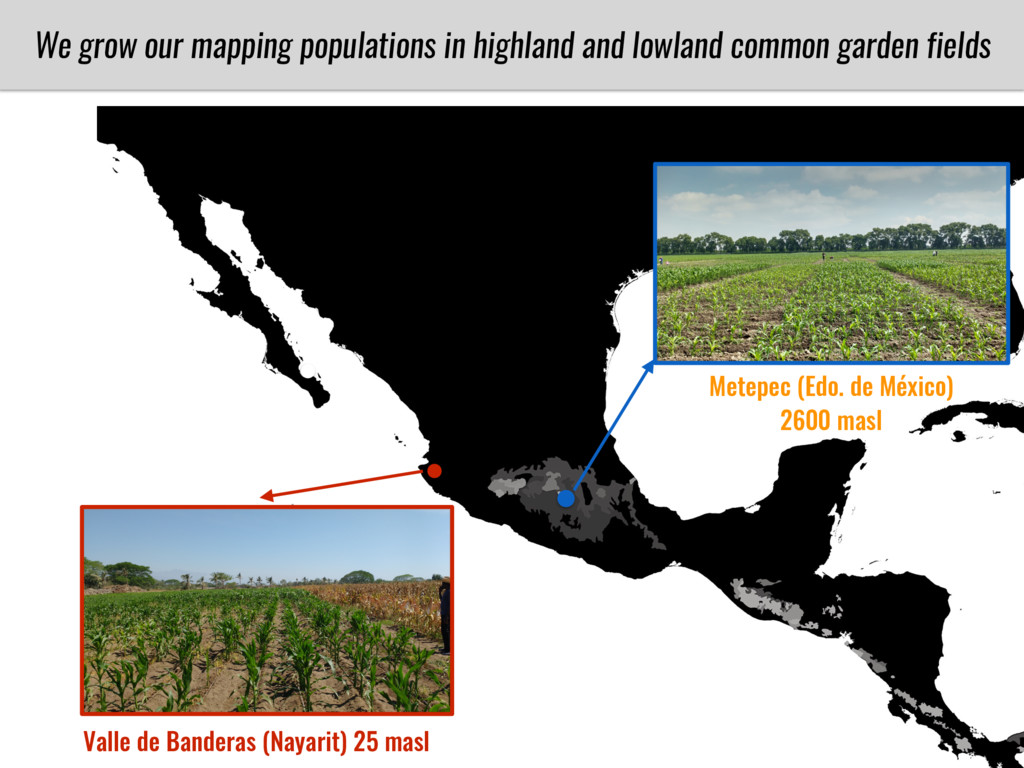
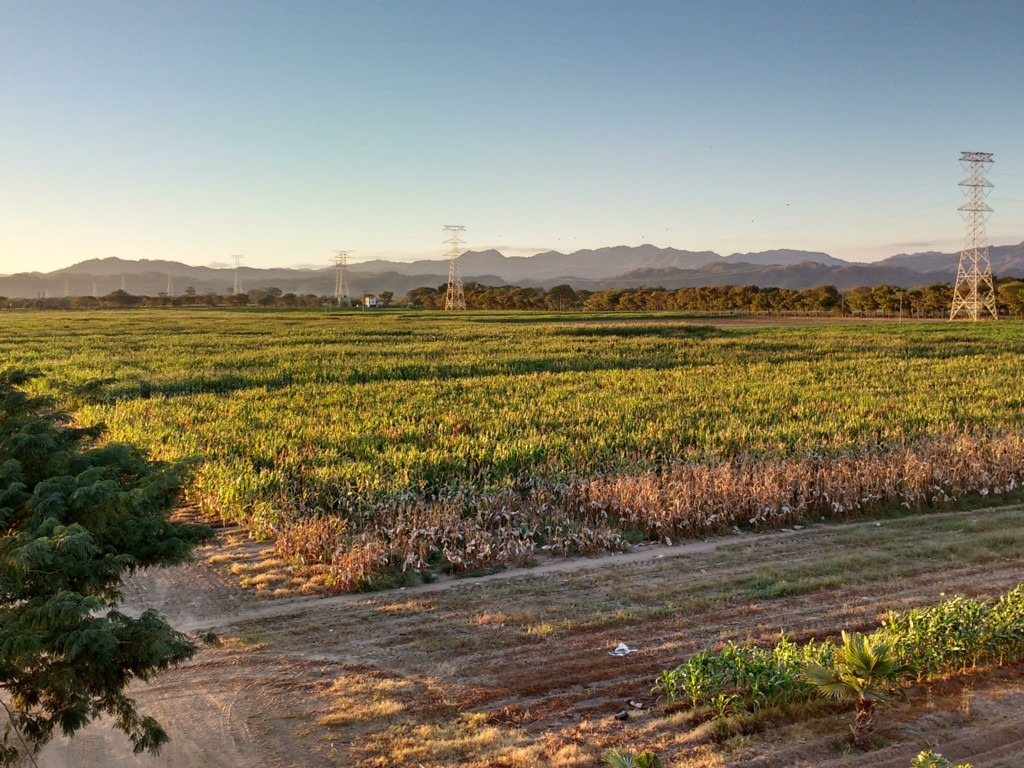
We grow our mapping populations in highland and lowland common
garden fields Valle de Banderas (Nayarit) 25 masl Metepec (Edo. de México) 2600 masl -
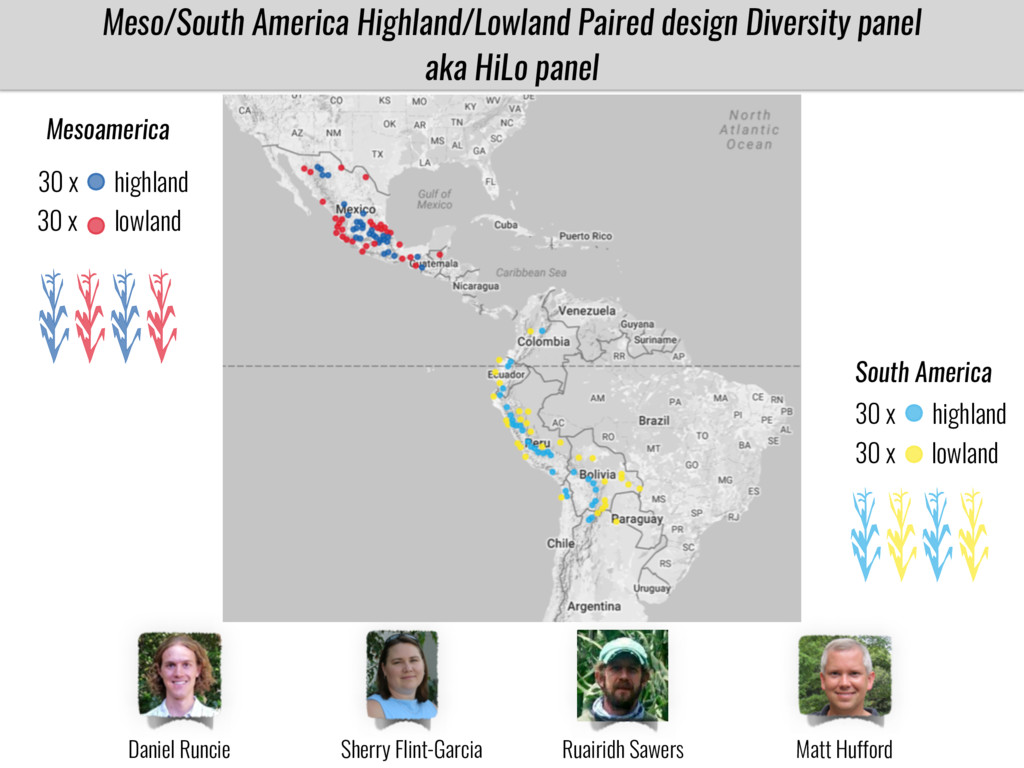
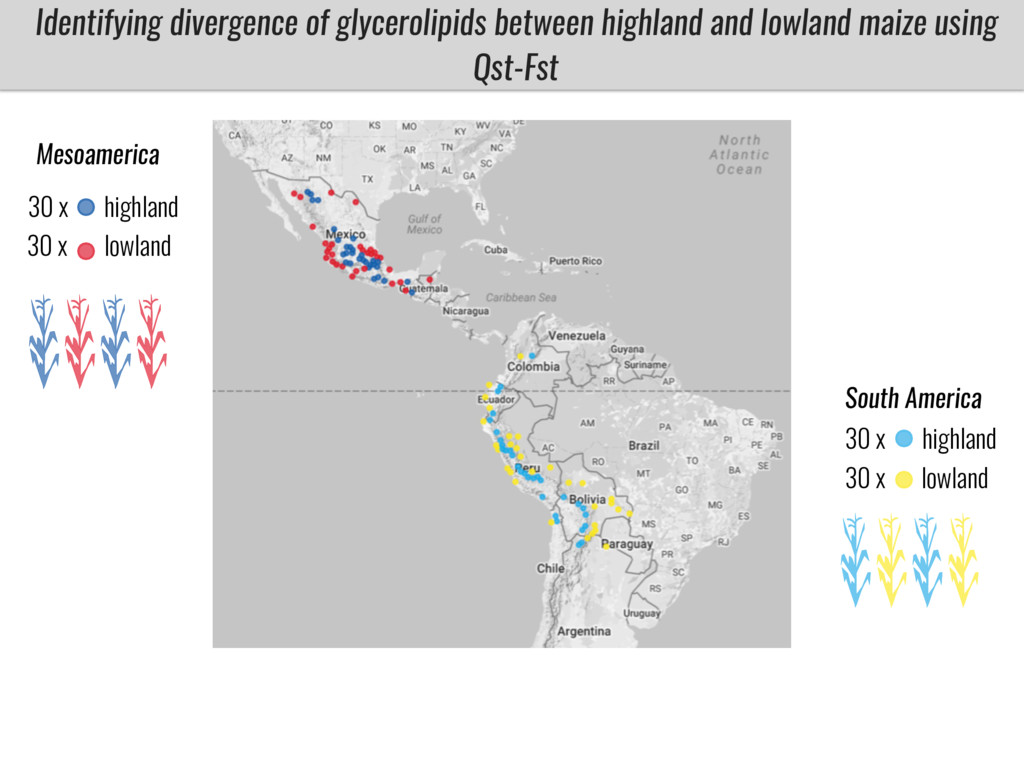
Meso/South America Highland/Lowland Paired design Diversity panel aka HiLo panel
Mesoamerica highland 30 x lowland 30 x highland 30 x lowland 30 x South America Daniel Runcie Matt Hufford Sherry Flint-Garcia Ruairidh Sawers -
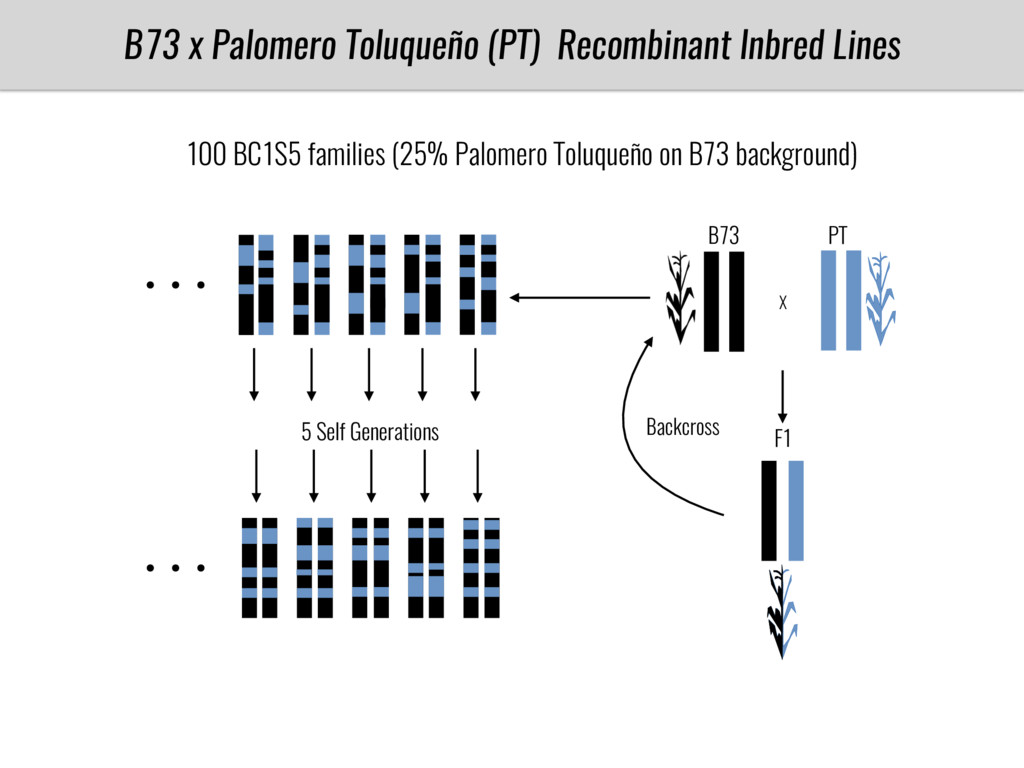
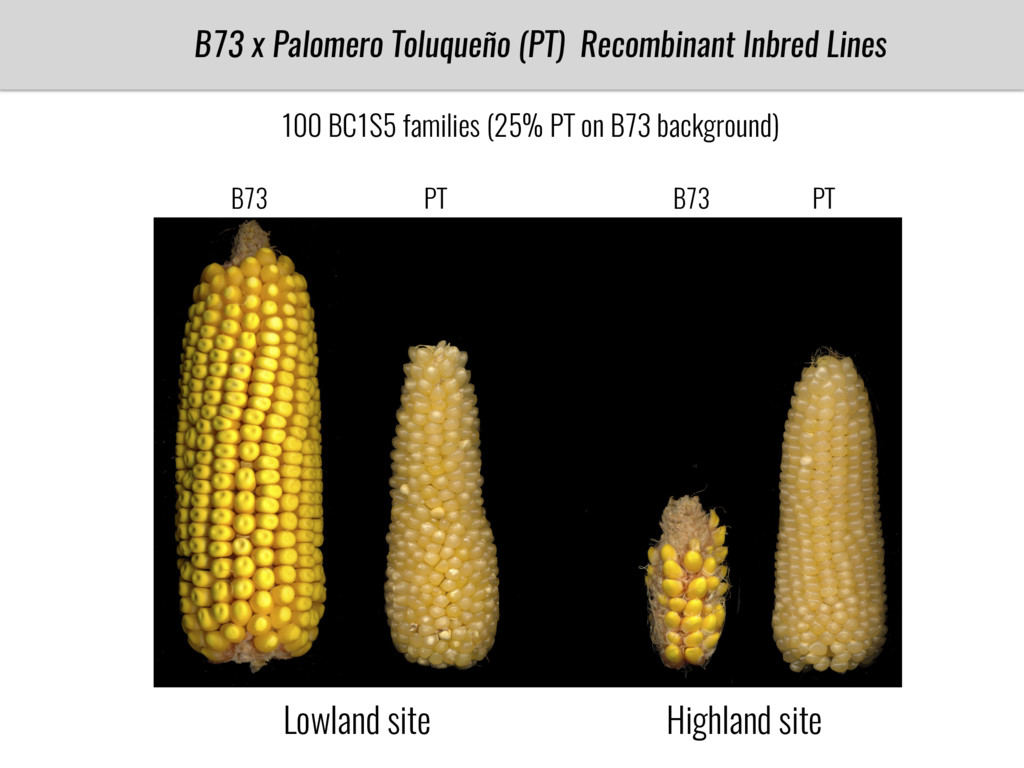
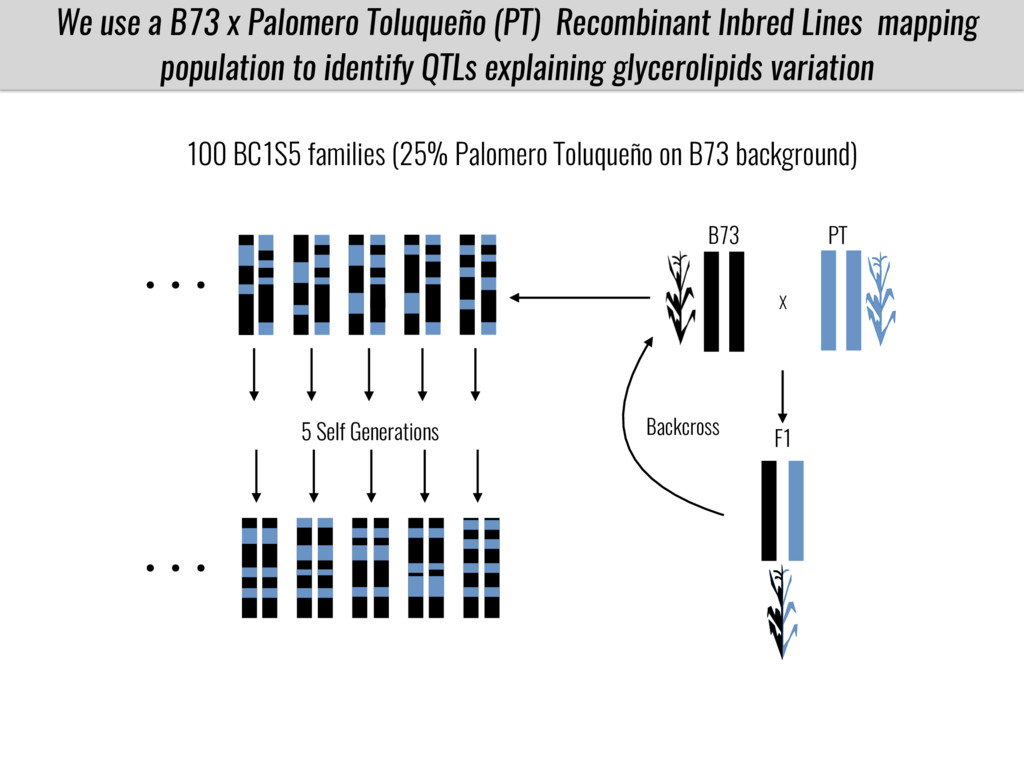
B73 x Palomero Toluqueño (PT) Recombinant Inbred Lines B73 PT
X F1 Backcross 100 BC1S5 families (25% Palomero Toluqueño on B73 background) 5 Self Generations -
B73 x Palomero Toluqueño (PT) Recombinant Inbred Lines 100 BC1S5
families (25% PT on B73 background) Lowland site Highland site B73 PT B73 PT LOWLAND Valle de Banderas (50masl) HIGHLAND Metepec (2600masl) Local adaptation drives maize diversity B73 B73 PT PT -
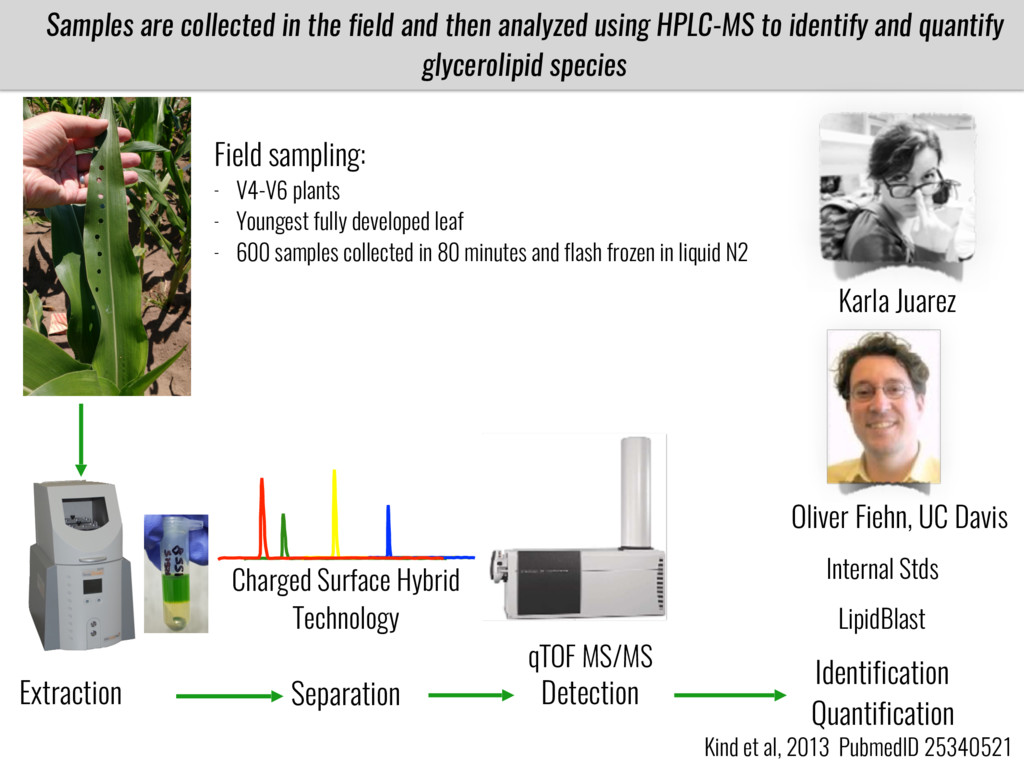
Separation Charged Surface Hybrid Technology Detection qTOF MS/MS Identification Quantification
Internal Stds LipidBlast Oliver Fiehn, UC Davis Samples are collected in the field and then analyzed using HPLC-MS to identify and quantify glycerolipid species Extraction Field sampling: - V4-V6 plants - Youngest fully developed leaf - 600 samples collected in 80 minutes and flash frozen in liquid N2 Kind et al, 2013 PubmedID 25340521 Karla Juarez -
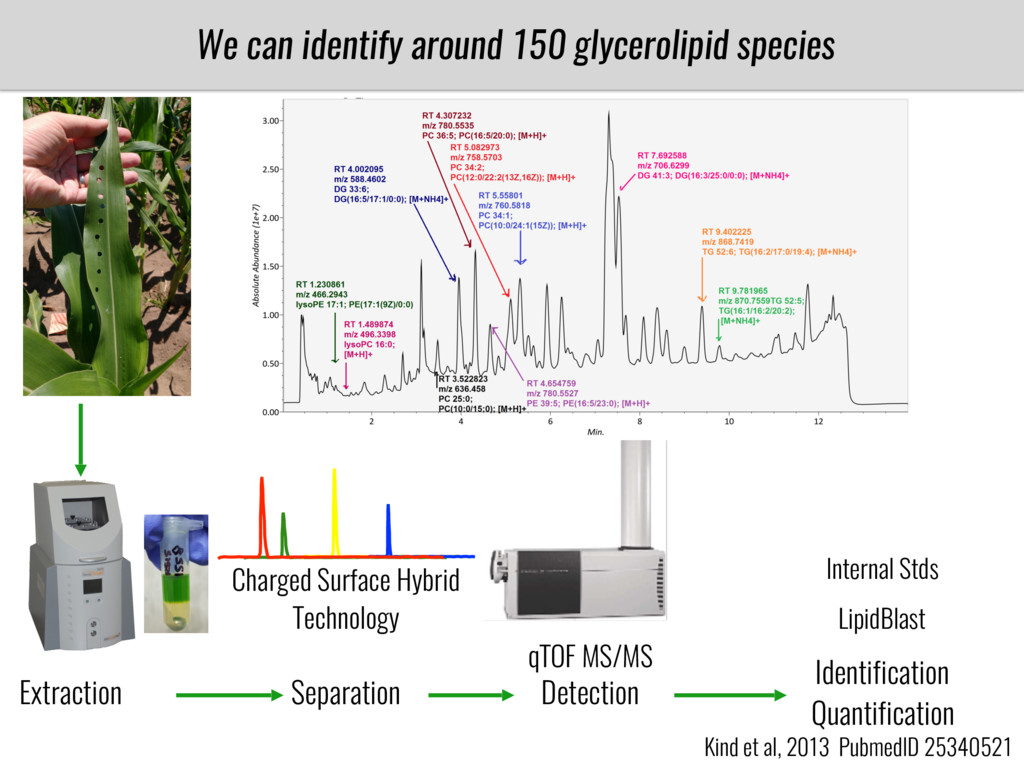
Separation Detection qTOF MS/MS Identification Quantification Internal Stds LipidBlast We
can identify around 150 glycerolipid species Extraction Kind et al, 2013 PubmedID 25340521 Charged Surface Hybrid Technology -
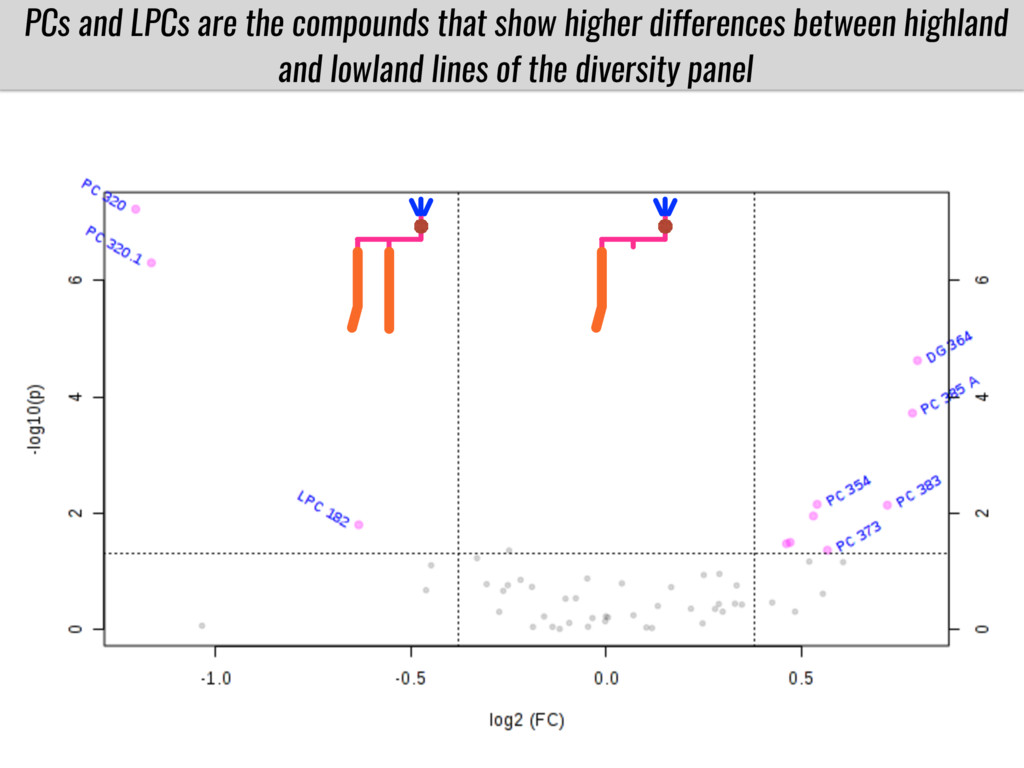
PCs and LPCs are the compounds that show higher differences
between highland and lowland lines of the diversity panel haring metabolomic features B) -
PCs and LPCs are the species that show higher differences
between highland and lowland lines, but we can see some differences between Meso and South America Mesoamerica South America Low High Low High Low High Low High Mesoamerica South America Meso_high SA_high Meso_low SA_low -
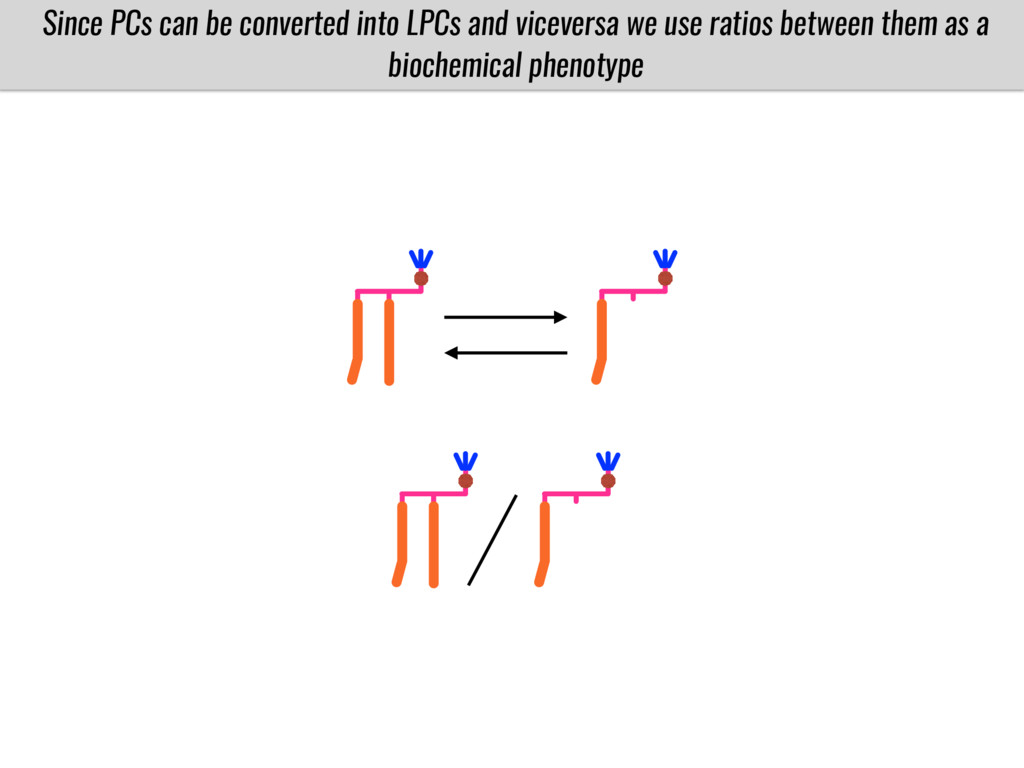
Since PCs can be converted into LPCs and viceversa we
use ratios between them as a biochemical phenotype -
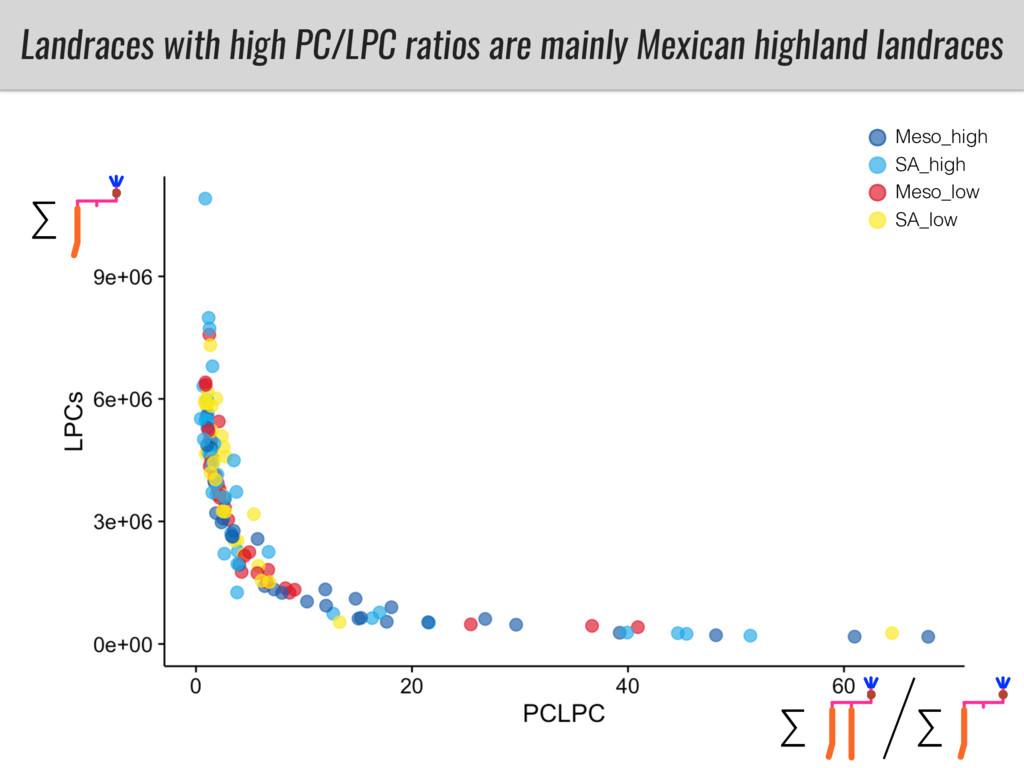
Landraces with high PC/LPC ratios are mainly Mexican highland landraces
∑ ∑ ∑ Meso_high SA_high Meso_low SA_low -
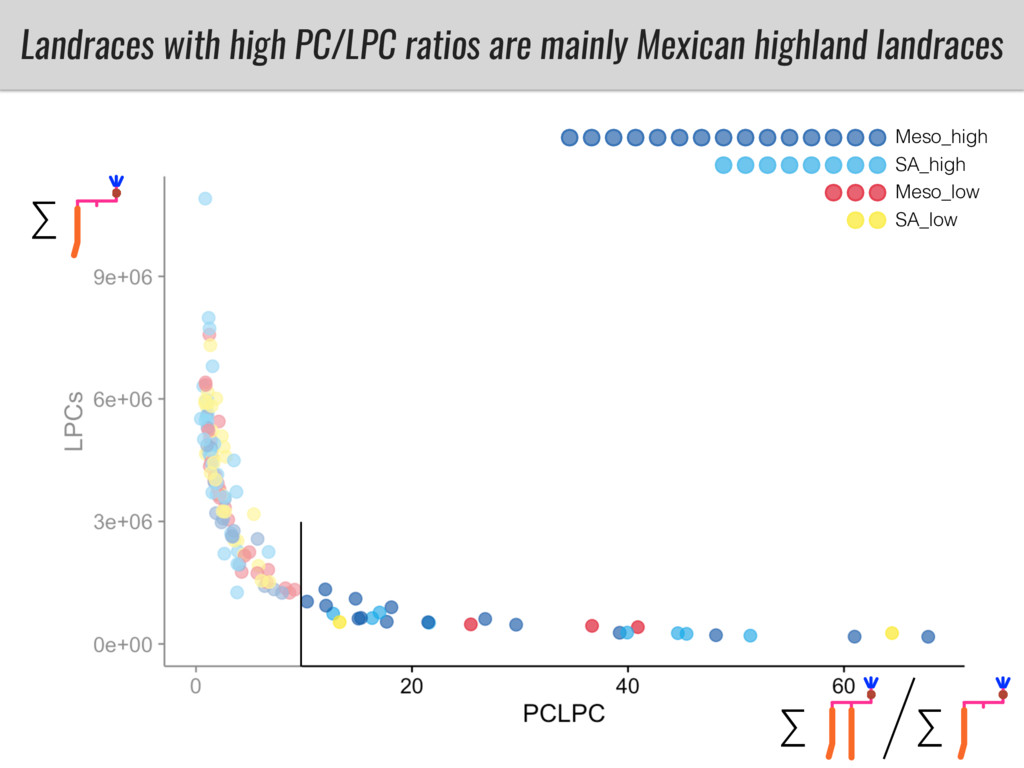
Landraces with high PC/LPC ratios are mainly Mexican highland landraces
∑ Meso_high SA_high Meso_low SA_low ∑ ∑ Meso_high SA_high Meso_low SA_low -
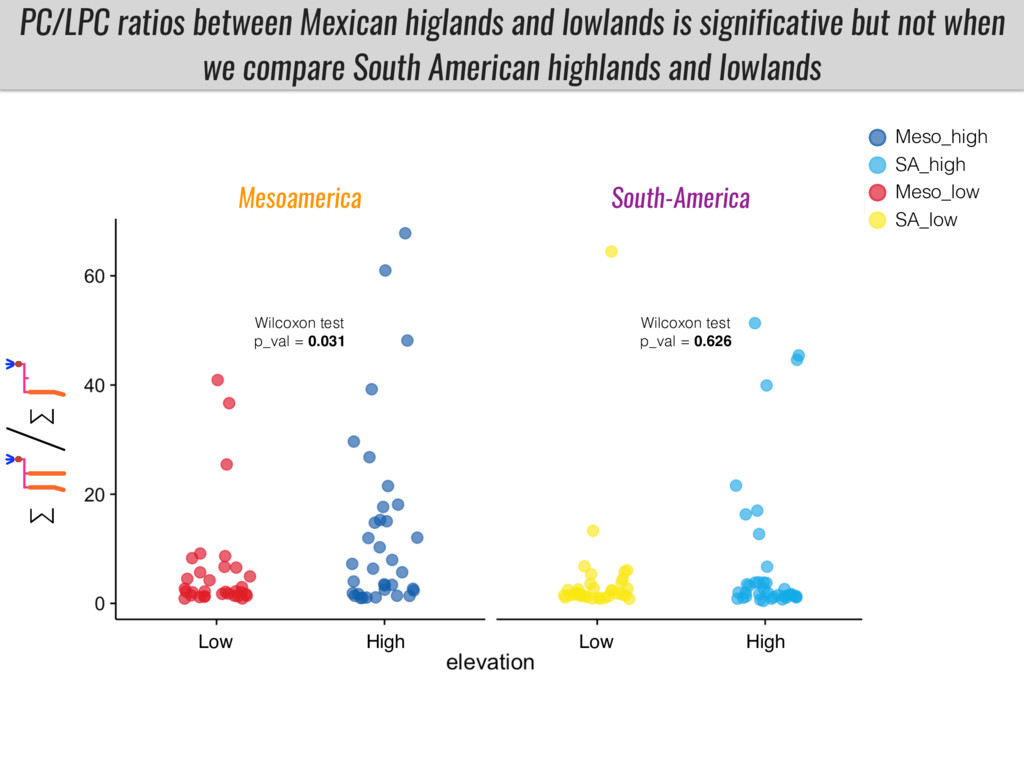
PC/LPC ratios between Mexican higlands and lowlands is significative but
not when we compare South American highlands and lowlands Meso_high SA_high Meso_low SA_low Mesoamerica South America ∑ ∑ Wilcoxon test p_val = 0.031 Low High Low High Wilcoxon test p_val = 0.626 Mesoamerica South-America -
We use a B73 x Palomero Toluqueño (PT) Recombinant Inbred
Lines mapping population to identify QTLs explaining glycerolipids variation B73 PT X F1 Backcross 100 BC1S5 families (25% Palomero Toluqueño on B73 background) 5 Self Generations -
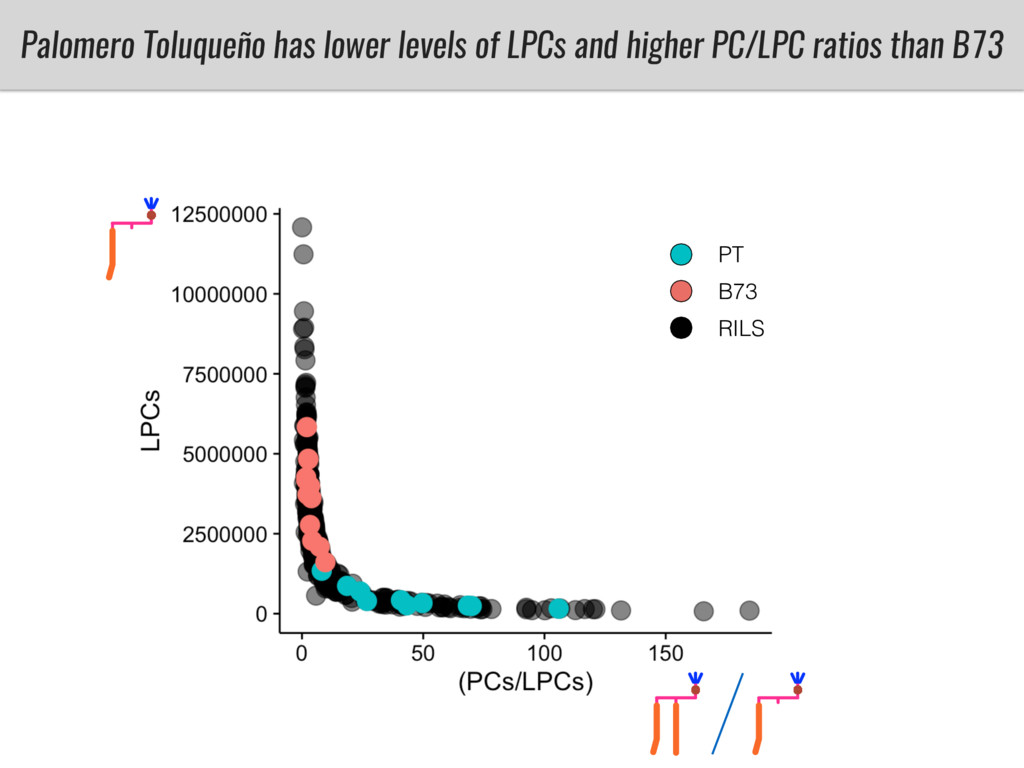
Palomero Toluqueño has lower levels of LPCs and higher PC/LPC
ratios than B73 PT RILS B73 -
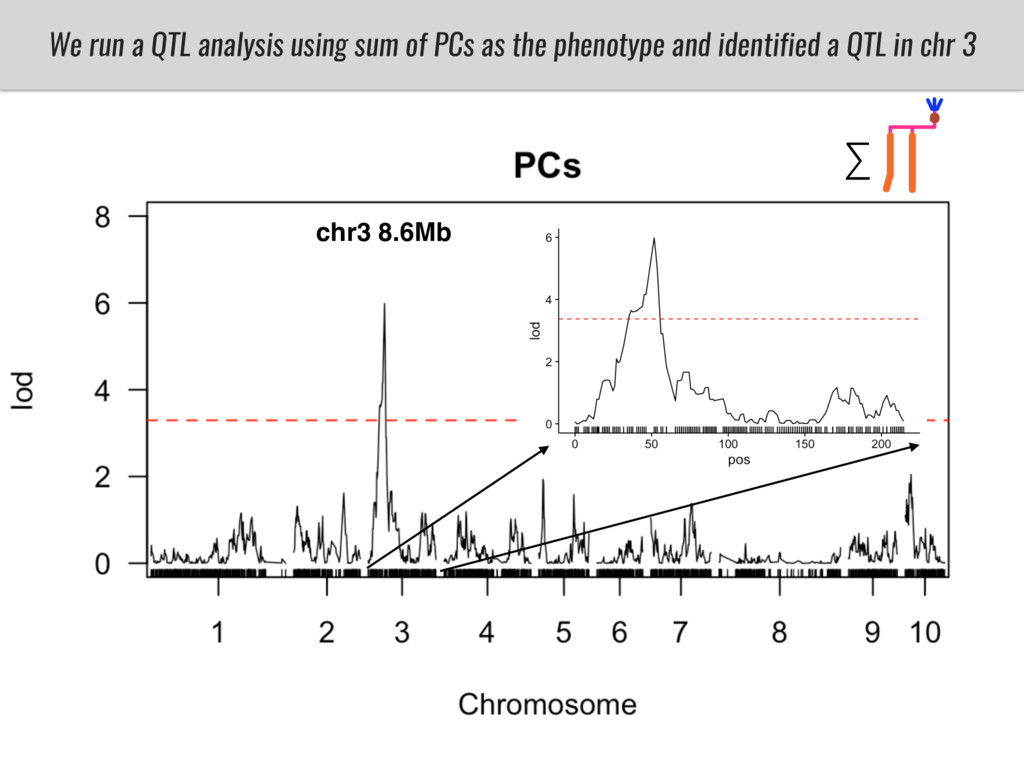
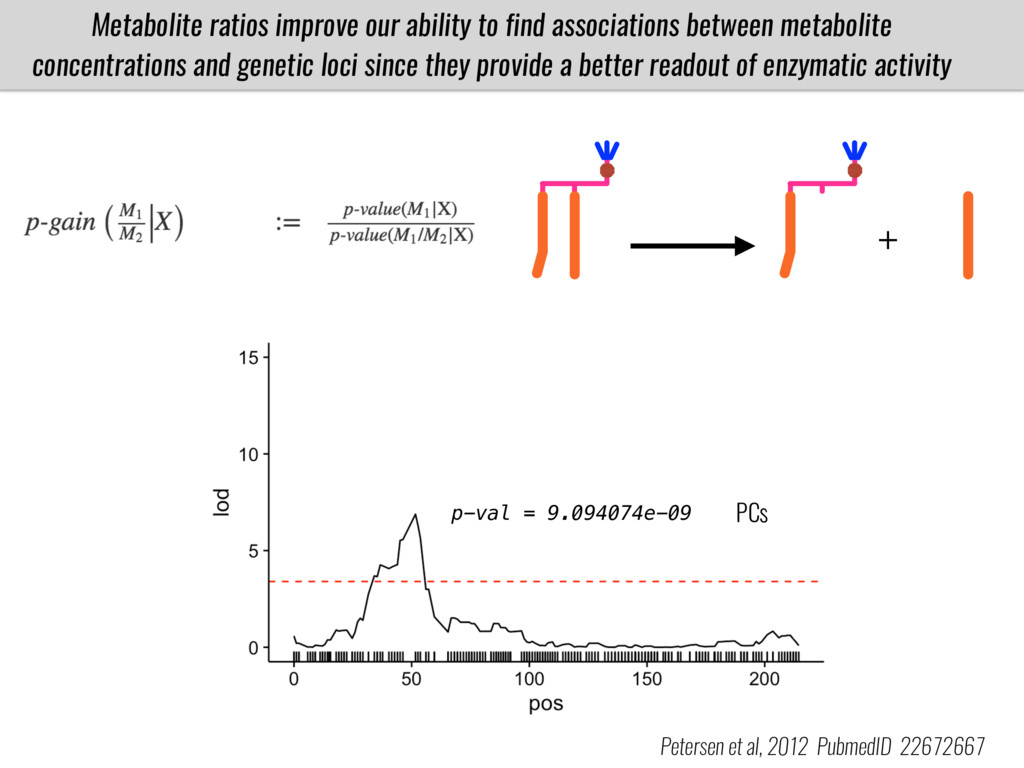
We run a QTL analysis using sum of PCs as
the phenotype and identified a QTL in chr 3 chr3 8.6Mb ∑ -
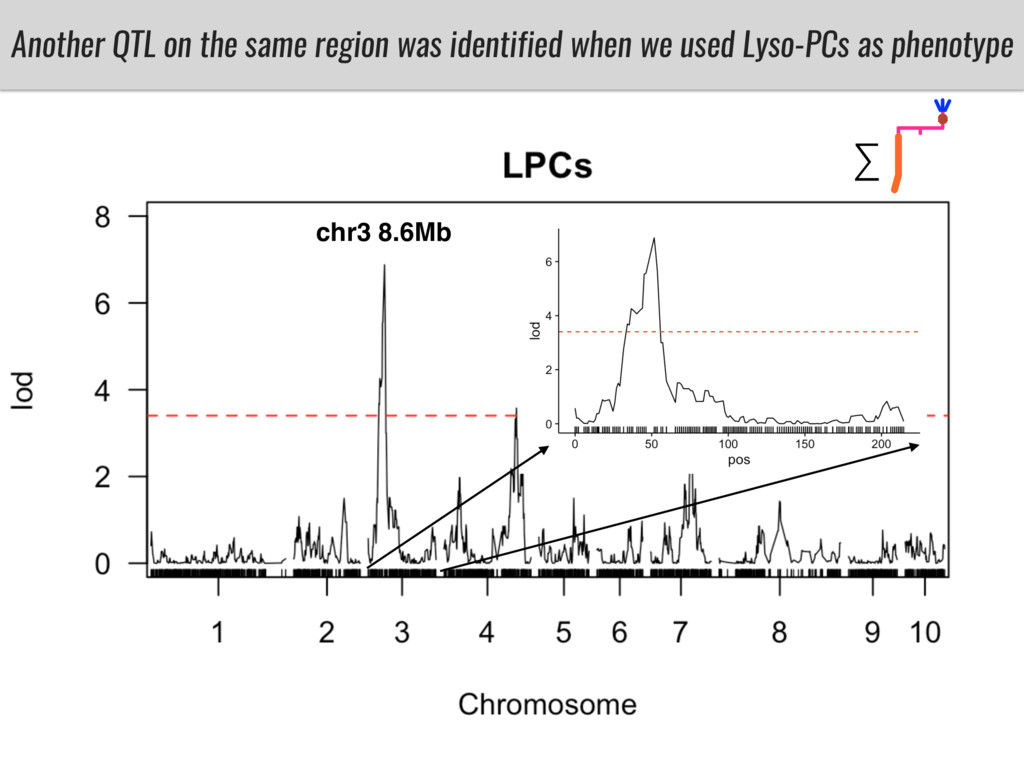
Another QTL on the same region was identified when we
used Lyso-PCs as phenotype chr3 8.6Mb ∑ -
Petersen et al, 2012 PubmedID 22672667 p-val = 9.094074e-09 PCs
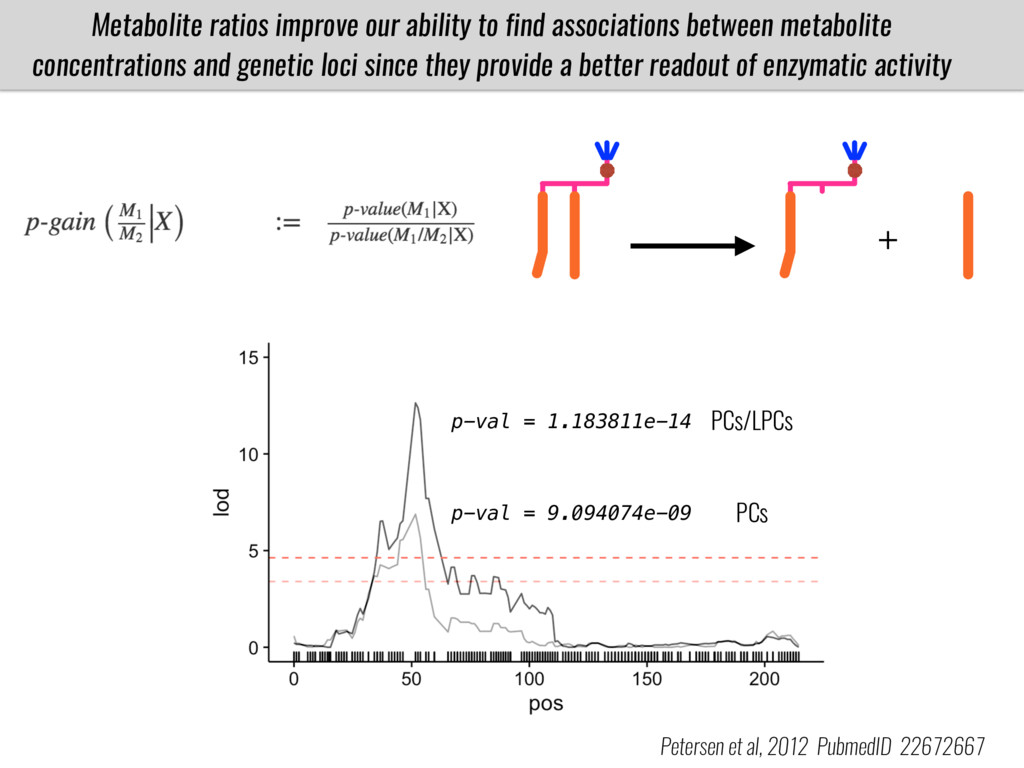
Metabolite ratios improve our ability to find associations between metabolite concentrations and genetic loci since they provide a better readout of enzymatic activity + -
Metabolite ratios improve our ability to find associations between metabolite
concentrations and genetic loci since they provide a better readout of enzymatic activity p-val = 9.094074e-09 p-val = 1.183811e-14 PCs PCs/LPCs Petersen et al, 2012 PubmedID 22672667 + -
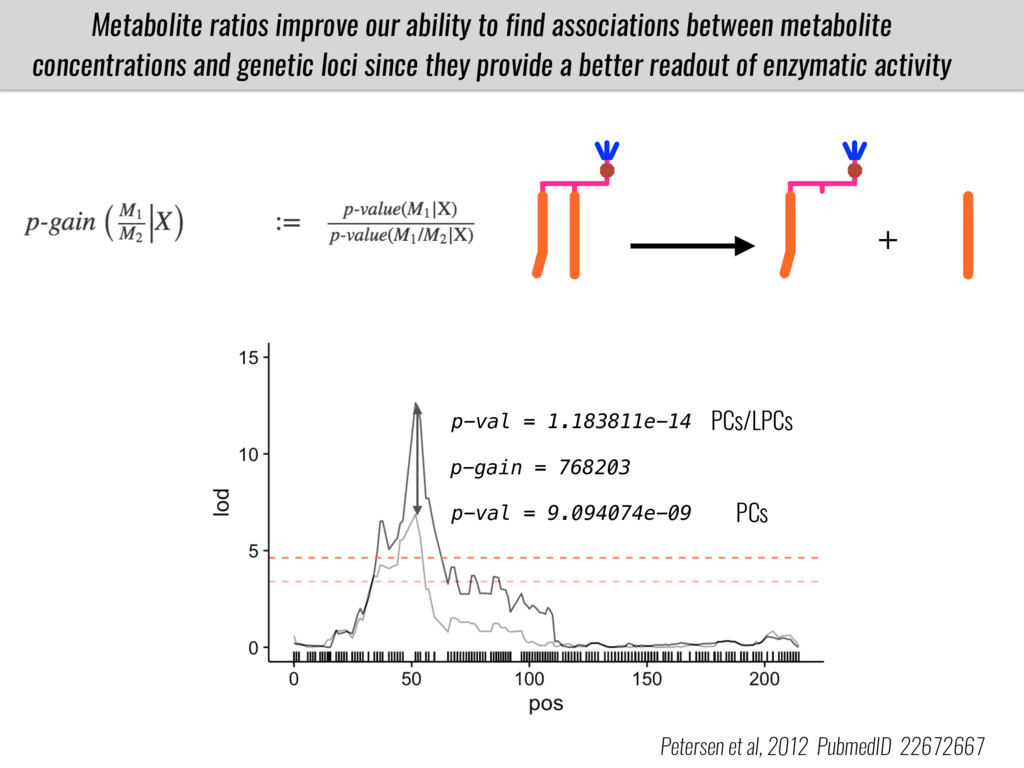
p-val = 9.094074e-09 p-val = 1.183811e-14 p-gain = 768203 PCs
PCs/LPCs Metabolite ratios improve our ability to find associations between metabolite concentrations and genetic loci since they provide a better readout of enzymatic activity Petersen et al, 2012 PubmedID 22672667 + -
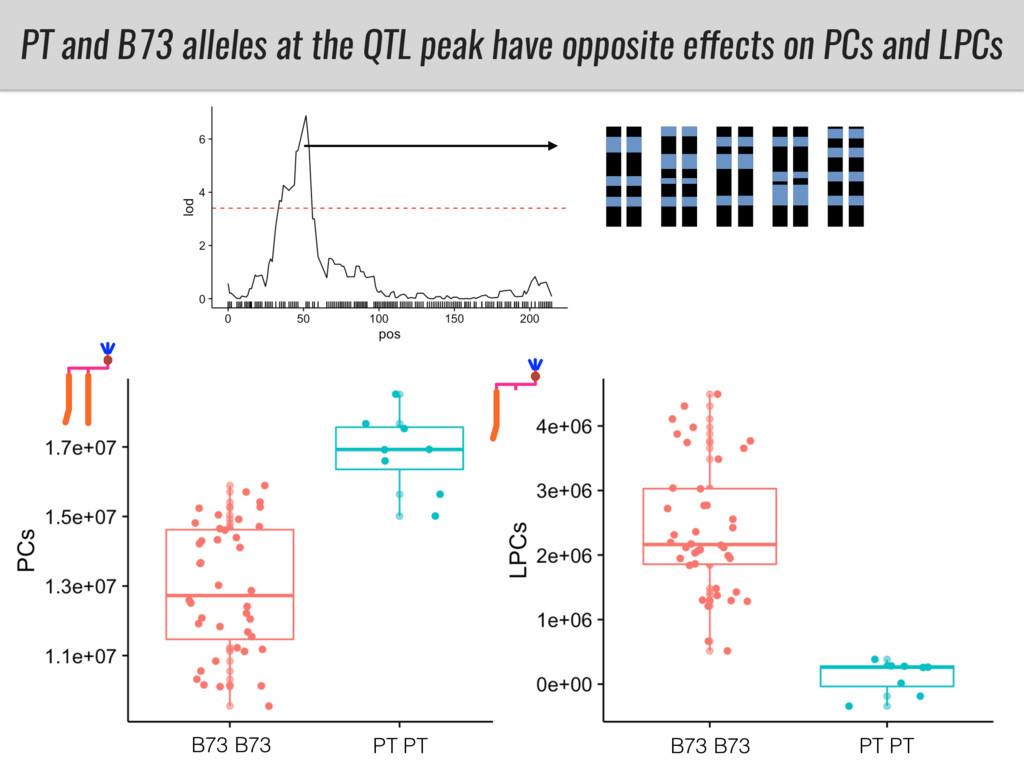
PT and B73 alleles at the QTL peak have opposite
effects on PCs and LPCs B73 B73 PT PT B73 B73 PT PT -
Heterozygous phenotype shows that the B73 allele is dominant B73
B73 PT PT B73 PT -
Is there any candidate gene in that region that makes
sense with our biochemical phenotype? -
A phospholipase A1 with predicted PC to lyso-PC activity is
right at the QTL peak GRMZM2G353444 + PLD PLC PLA1 PLA2 -
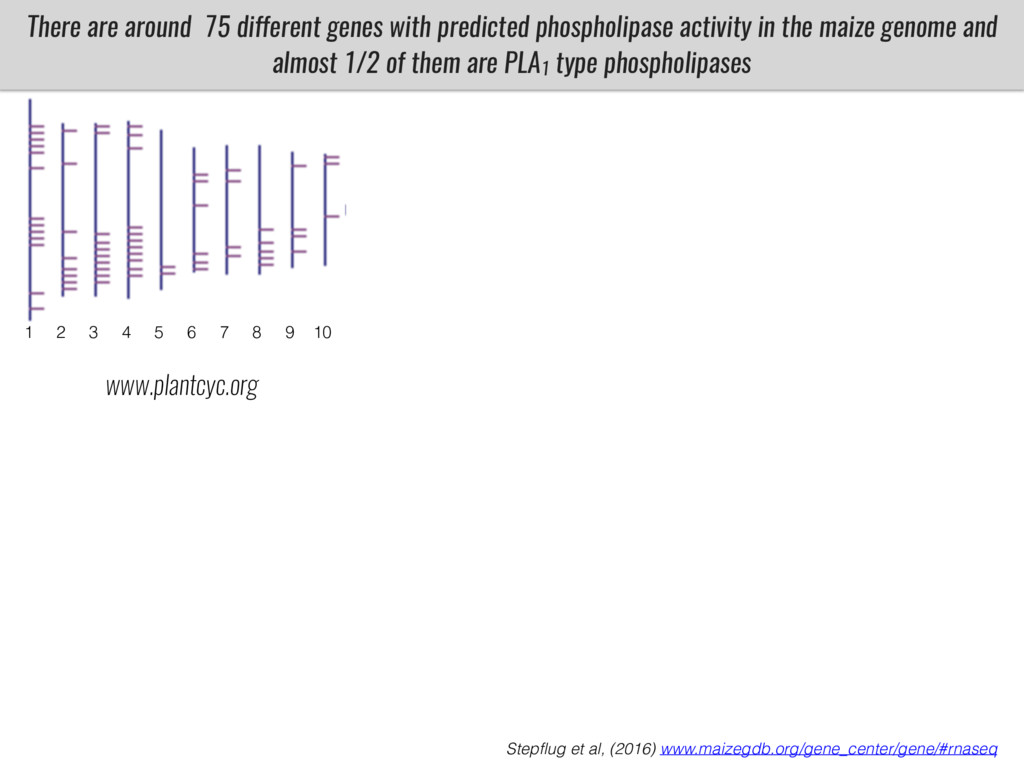
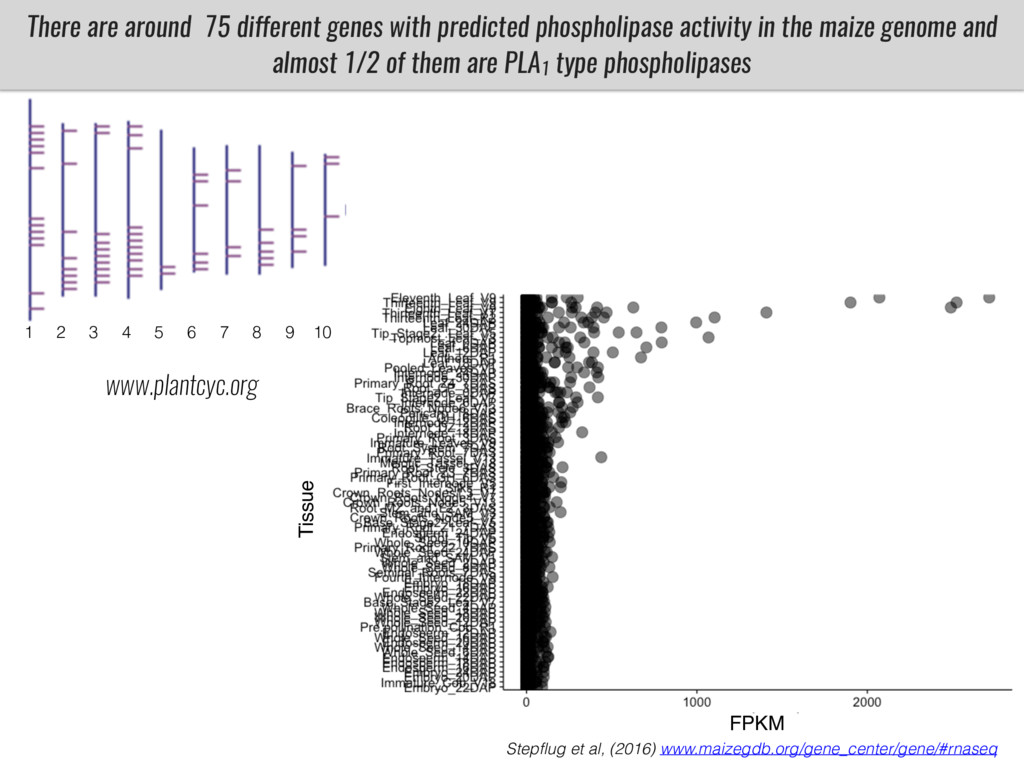
There are around 75 different genes with predicted phospholipase activity
in the maize genome and almost 1/2 of them are PLA1 type phospholipases Stepflug et al, (2016) www.maizegdb.org/gene_center/gene/#rnaseq www.plantcyc.org 1 2 3 4 5 6 7 8 9 10 -
There are around 75 different genes with predicted phospholipase activity
in the maize genome and almost 1/2 of them are PLA1 type phospholipases Stepflug et al, (2016) www.maizegdb.org/gene_center/gene/#rnaseq Tissue FPKM www.plantcyc.org 1 2 3 4 5 6 7 8 9 10 -
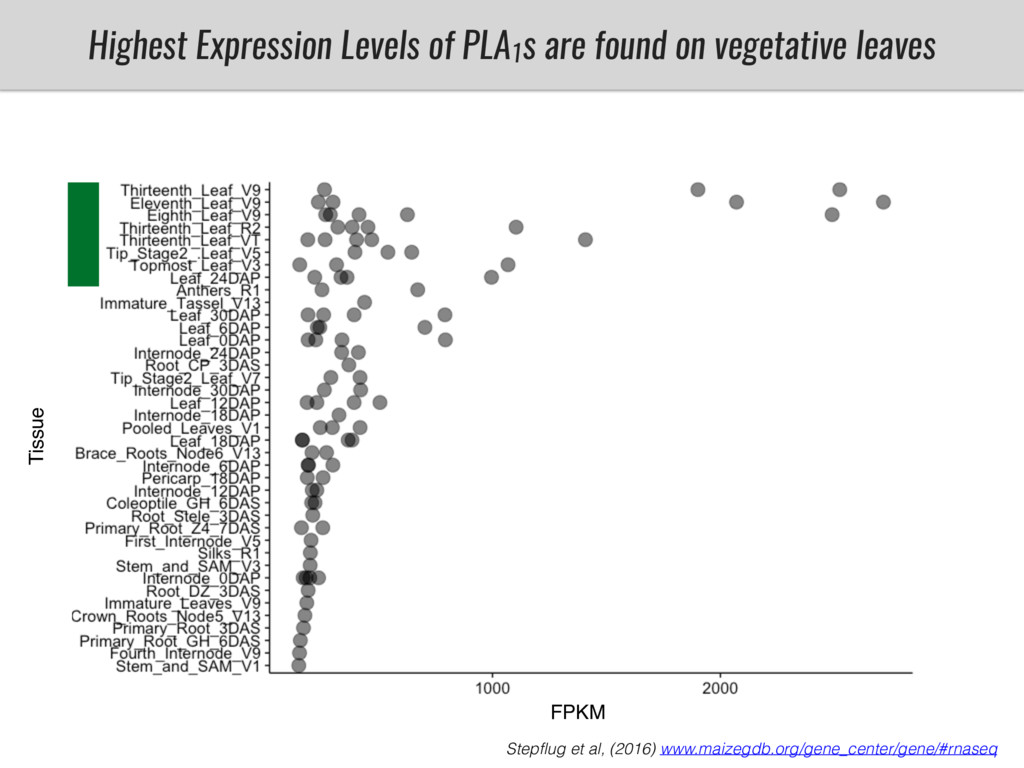
Highest Expression Levels of PLA1 s are found on vegetative
leaves Tissue FPKM Stepflug et al, (2016) www.maizegdb.org/gene_center/gene/#rnaseq -
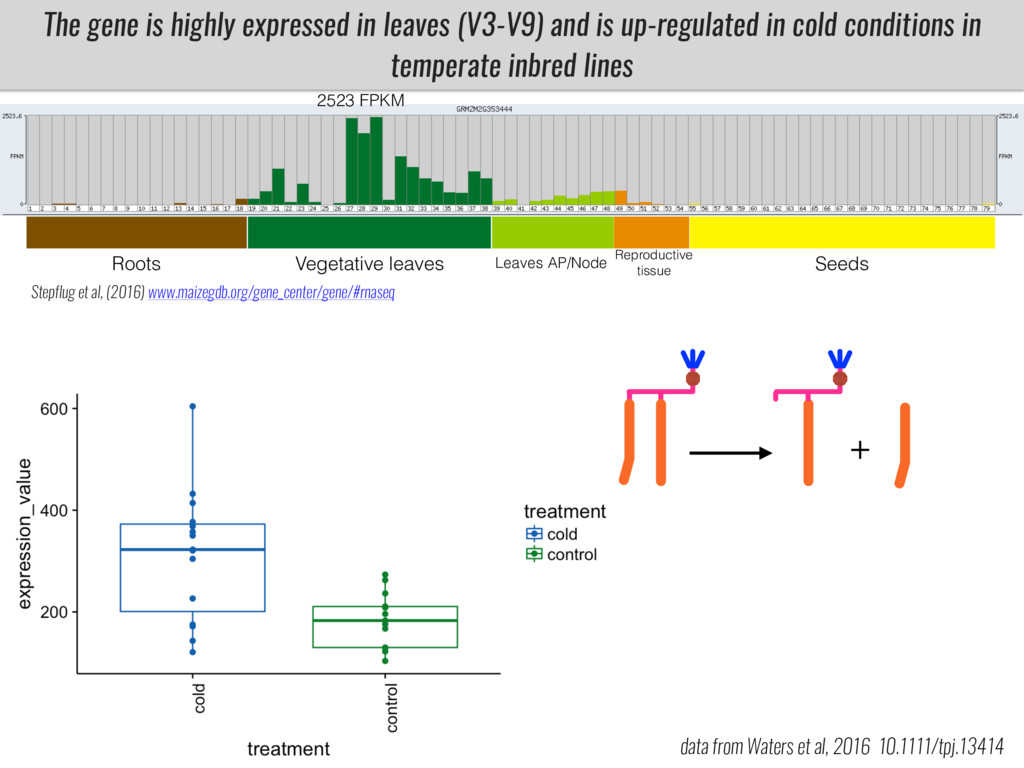
The candidate gene is one of the most highly expressed
PLA1 s GRMZM2G353444 Tissue FPKM Stepflug et al, (2016) www.maizegdb.org/gene_center/gene/#rnaseq -
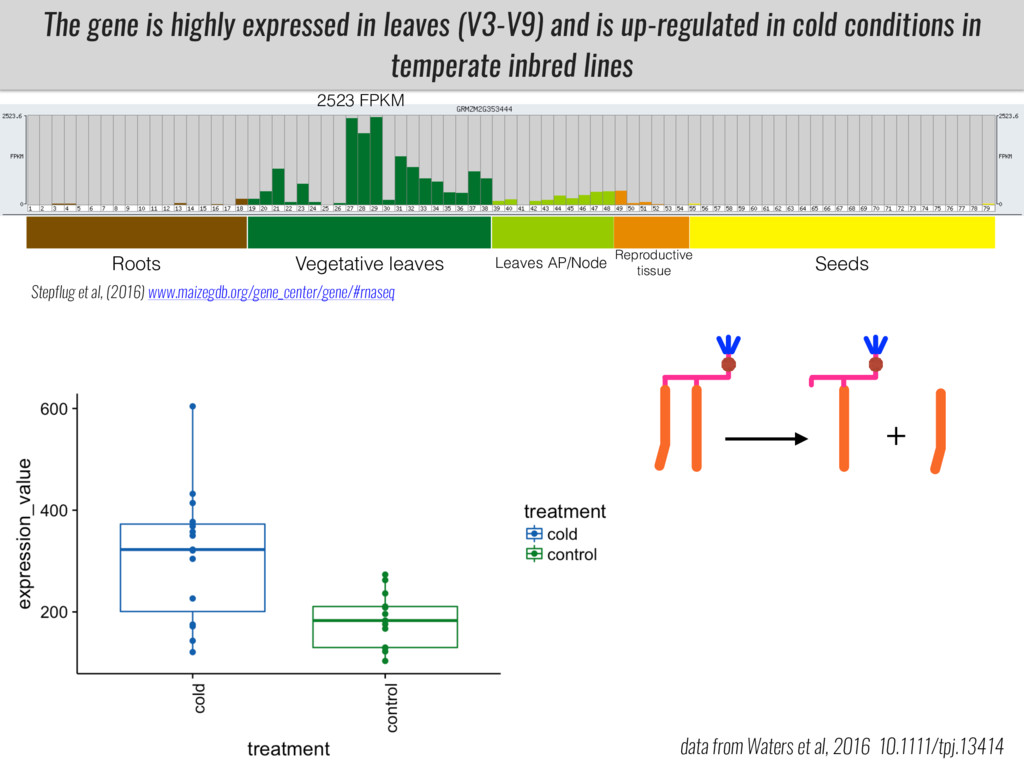
The gene is highly expressed in leaves (V3-V9) and is
up-regulated in cold conditions in temperate inbred lines 2523 FPKM Roots Vegetative leaves Leaves AP/Node Reproductive tissue Seeds Stepflug et al, (2016) www.maizegdb.org/gene_center/gene/#rnaseq data from Waters et al, 2016 10.1111/tpj.13414 + -
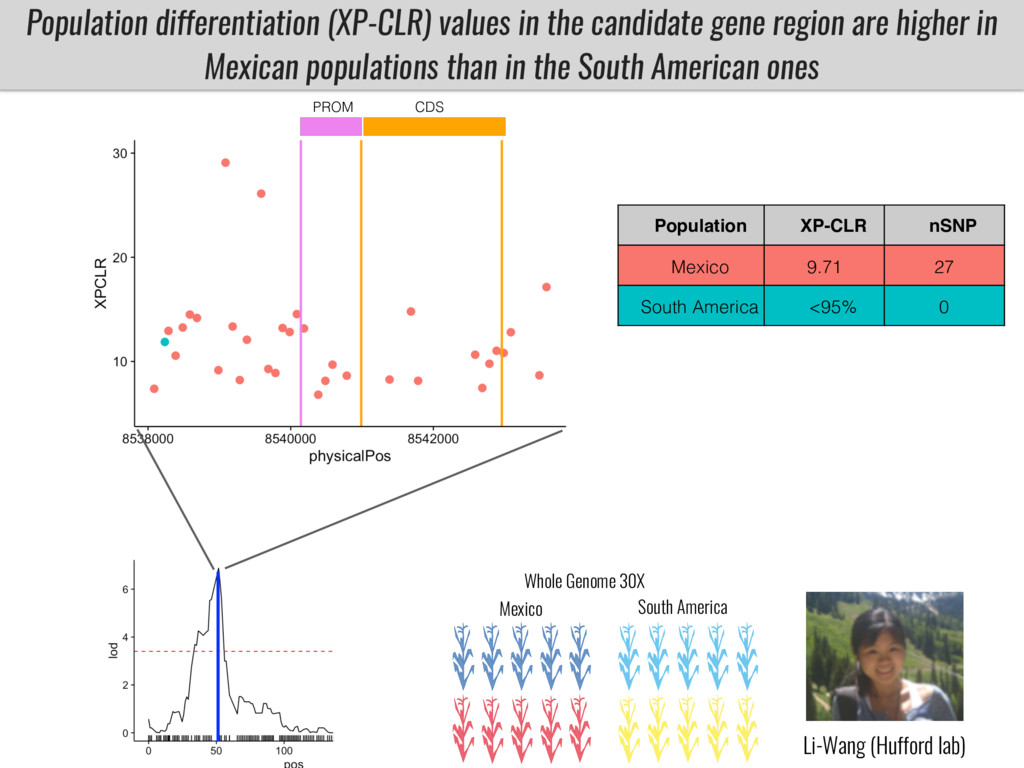
Population differentiation (XP-CLR) values in the candidate gene region are
higher in Mexican populations than in the South American ones CDS PROM Population XP-CLR nSNP Mexico 9.71 27 South America <95% 0 Li-Wang (Hufford lab) Mexico South America Whole Genome 30X -
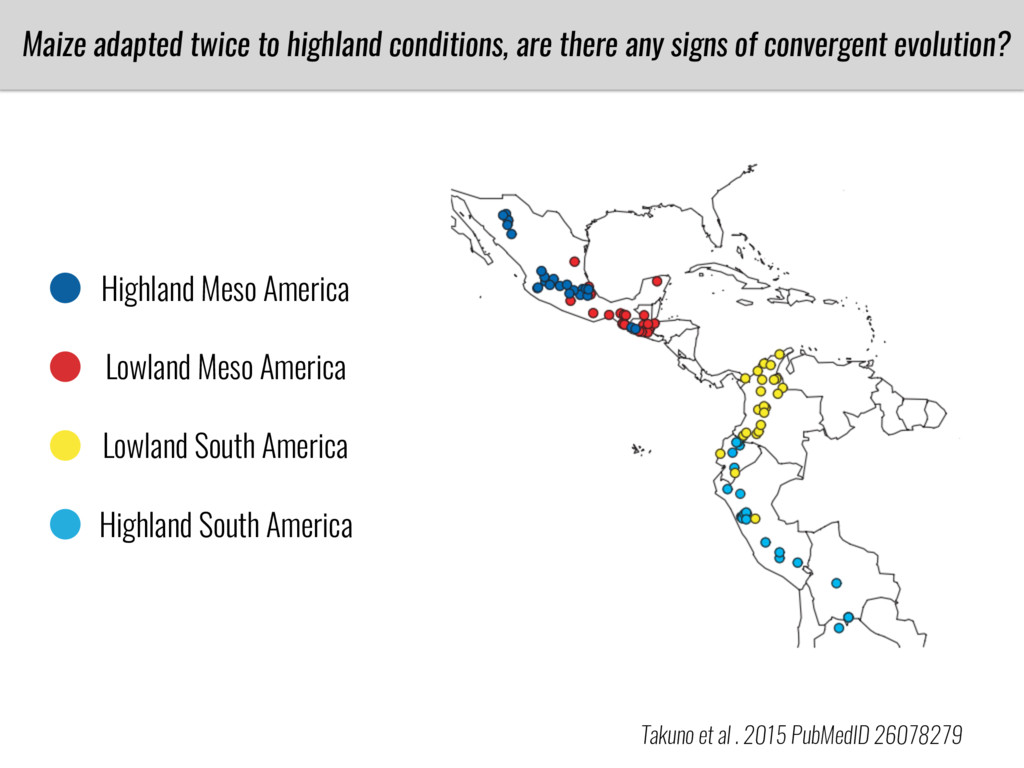
Maize adapted twice to highland conditions, are there any signs
of convergent evolution? Lowland Meso America Lowland South America Highland South America Highland Meso America Takuno et al . 2015 PubMedID 26078279 -
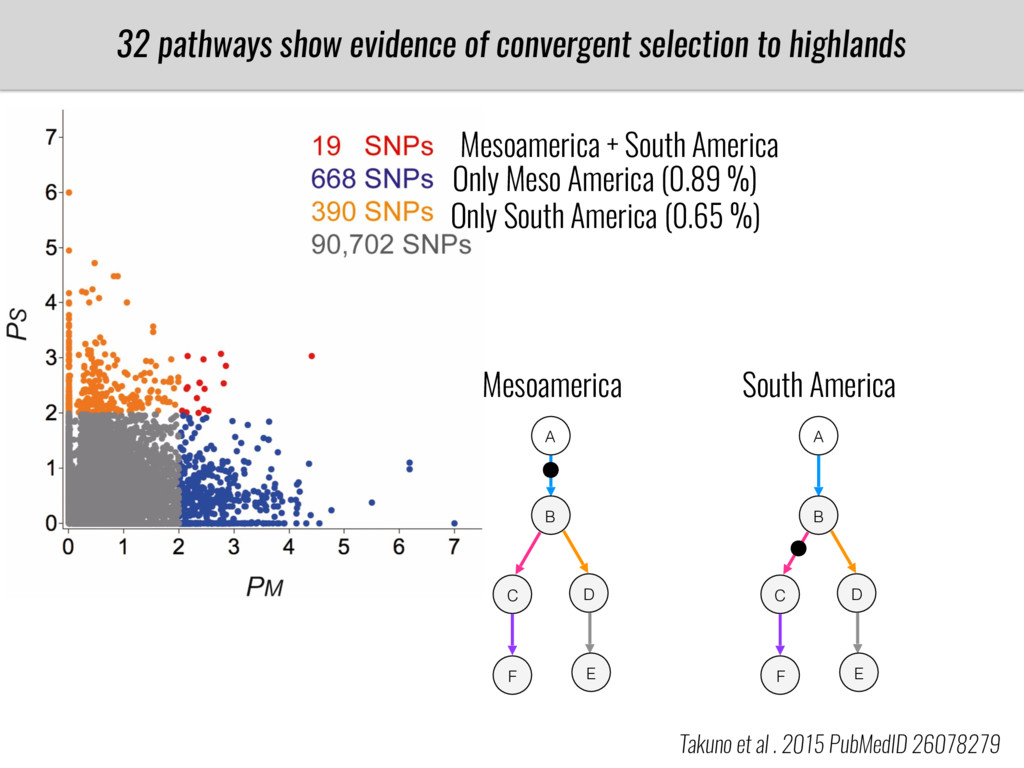
Very few genes show signs of convergent highland adaptation between
Meso America and South America. Only Meso America (0.89 %) Only South America (0.65 %) Mesoamerica + South America Takuno et al . 2015 PubMedID 26078279 -
32 pathways show evidence of convergent selection to highlands Only
Meso America (0.89 %) Only South America (0.65 %) Mesoamerica + South America Takuno et al . 2015 PubMedID 26078279 A B C D E F A B C D E F Mesoamerica South America -
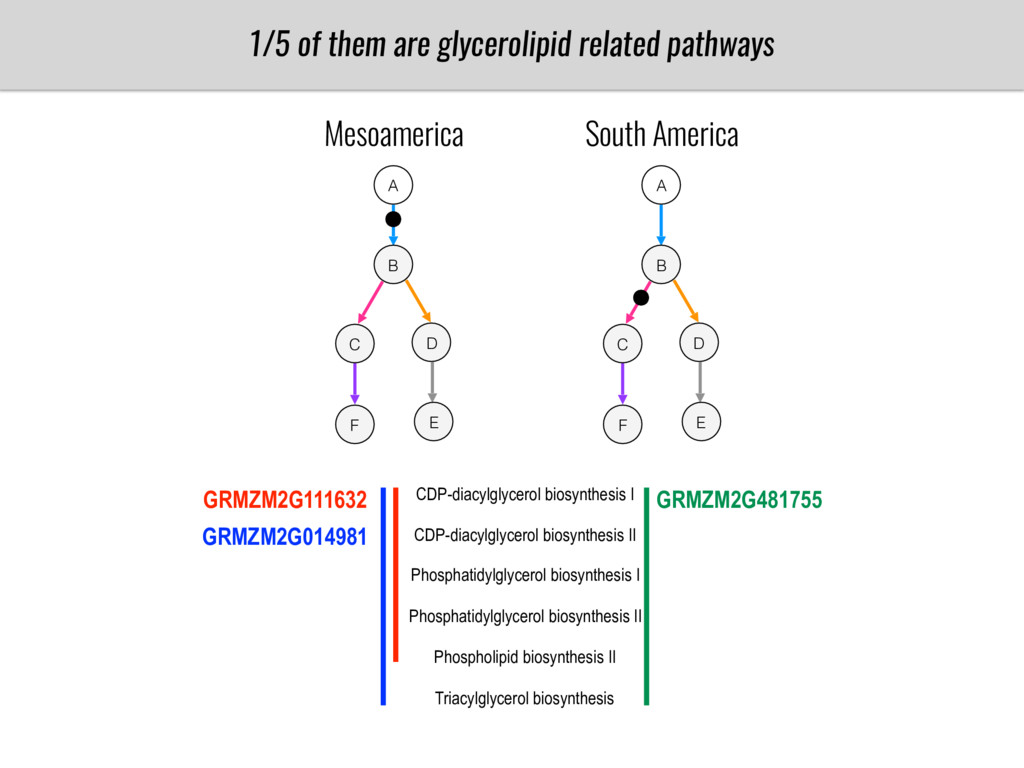
1/5 of them are glycerolipid related pathways GRMZM2G014981 GRMZM2G111632 GRMZM2G481755
CDP-diacylglycerol biosynthesis I CDP-diacylglycerol biosynthesis II Phosphatidylglycerol biosynthesis I Phosphatidylglycerol biosynthesis II Phospholipid biosynthesis II Triacylglycerol biosynthesis A B C D E F A B C D E F Mesoamerica South America -
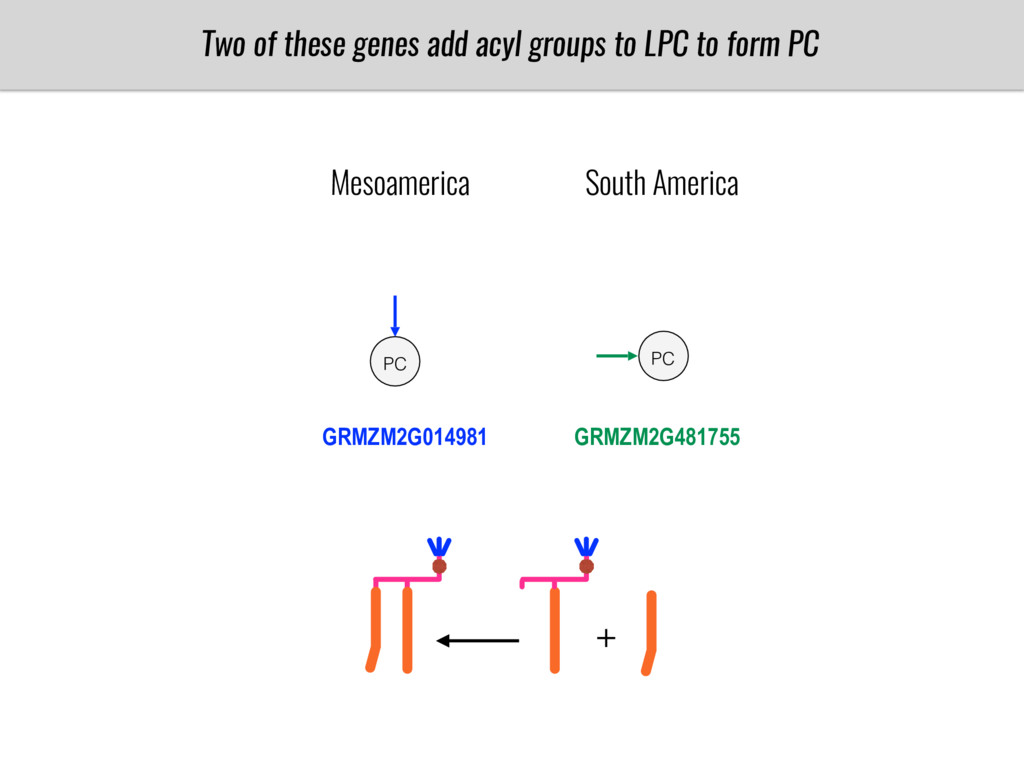
Two of these genes add acyl groups to LPC to
form PC GRMZM2G014981 GRMZM2G481755 PC Mesoamerica South America PC + -
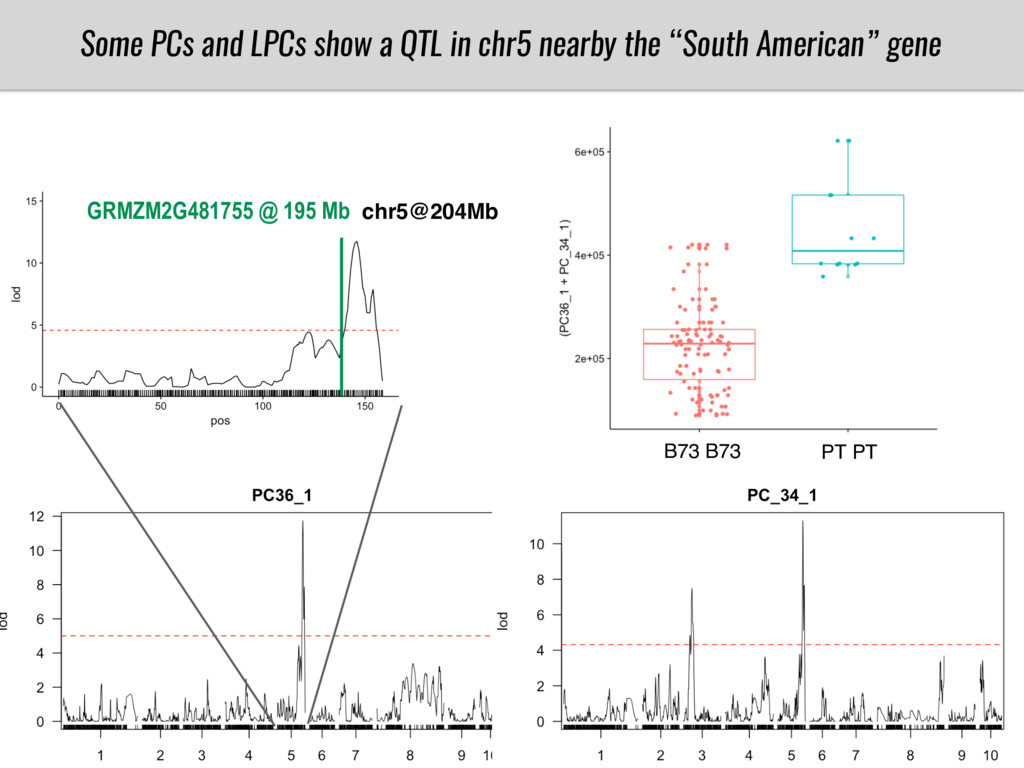
Some PCs and LPCs show a QTL in chr5 nearby
the “South American” gene chr5@204Mb GRMZM2G481755 @ 195 Mb B73 B73 PT PT -
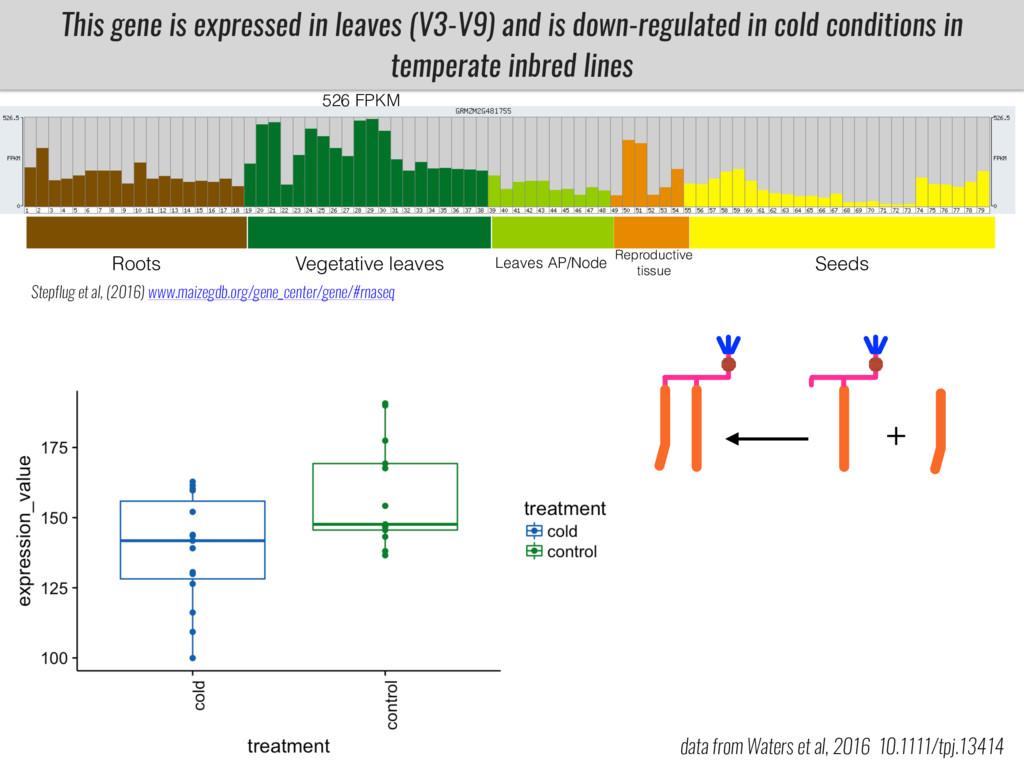
This gene is expressed in leaves (V3-V9) and is down-regulated
in cold conditions in temperate inbred lines Roots Vegetative leaves Leaves AP/Node Reproductive tissue Seeds Stepflug et al, (2016) www.maizegdb.org/gene_center/gene/#rnaseq data from Waters et al, 2016 10.1111/tpj.13414 526 FPKM + -
The gene is highly expressed in leaves (V3-V9) and is
up-regulated in cold conditions in temperate inbred lines 2523 FPKM Roots Vegetative leaves Leaves AP/Node Reproductive tissue Seeds Stepflug et al, (2016) www.maizegdb.org/gene_center/gene/#rnaseq data from Waters et al, 2016 10.1111/tpj.13414 + -
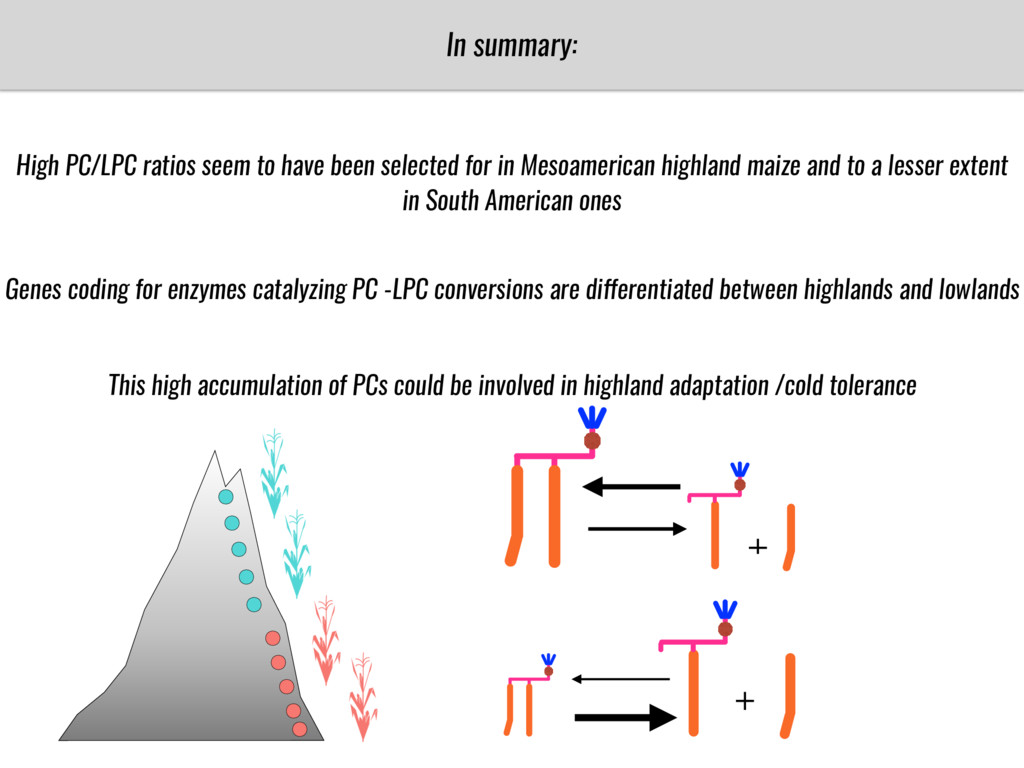
In summary: High PC/LPC ratios seem to have been selected
for in Mesoamerican highland maize and to a lesser extent in South American ones Genes coding for enzymes catalyzing PC -LPC conversions are differentiated between highlands and lowlands This high accumulation of PCs could be involved in highland adaptation /cold tolerance + + -
Currently working on: -Identifying possible mutations in the candidate gene
that could explain the biochemical phenotypes that we observe in B73/PT -
Currently working on: -Identifying possible mutations in the candidate gene
that could explain biochemical phenotypes that we observe in B73/PT -Developing markers for candidate gene(s) to explore phenotype-genotypes associations in diversity panels -
Currently working on: -Developing NILs and mutants of candidate genes
to test the possible effect of PT alleles on highland adaptation and under cold/low P conditions. -Identifying possible mutations in the candidate gene that could explain biochemical phenotypes that we observe in B73/PT -Developing markers for candidate gene(s) to explore phenotype-genotypes associations in diversity panels -
Currently working on: -Developing NILs and mutants of candidate genes
to test the possible effect of PT alleles on highland adaptation and under cold/low P conditions. -Identifying possible mutations in the candidate gene that could explain biochemical phenotypes that we observe in B73/PT -Developing markers for candidate gene(s) to explore phenotype-genotypes associations in diversity panels -Identifying divergence of glycerolipids between highland and lowland maize using Qst-Fst. -
Mesoamerica highland 30 x lowland 30 x highland 30 x
lowland 30 x South America Identifying divergence of glycerolipids between highland and lowland maize using Qst-Fst -
Currently working on: -Developing NILs and mutants of candidate genes
to test the possible effect of PT alleles on highland adaptation and under cold/low P conditions. -Identifying possible mutations in the candidate gene that could explain biochemical phenotypes that we observe in B73/PT -Developing markers for candidate gene(s) to explore phenotype-genotypes associations in diversity panels -Identifying divergence of glycerolipids between highland and lowland maize using Qst-Fst. -GWAS on glycerolipids and genes involved in glycerolipids pathways using RNA-Seq ASE on B73 x LRs F1s -
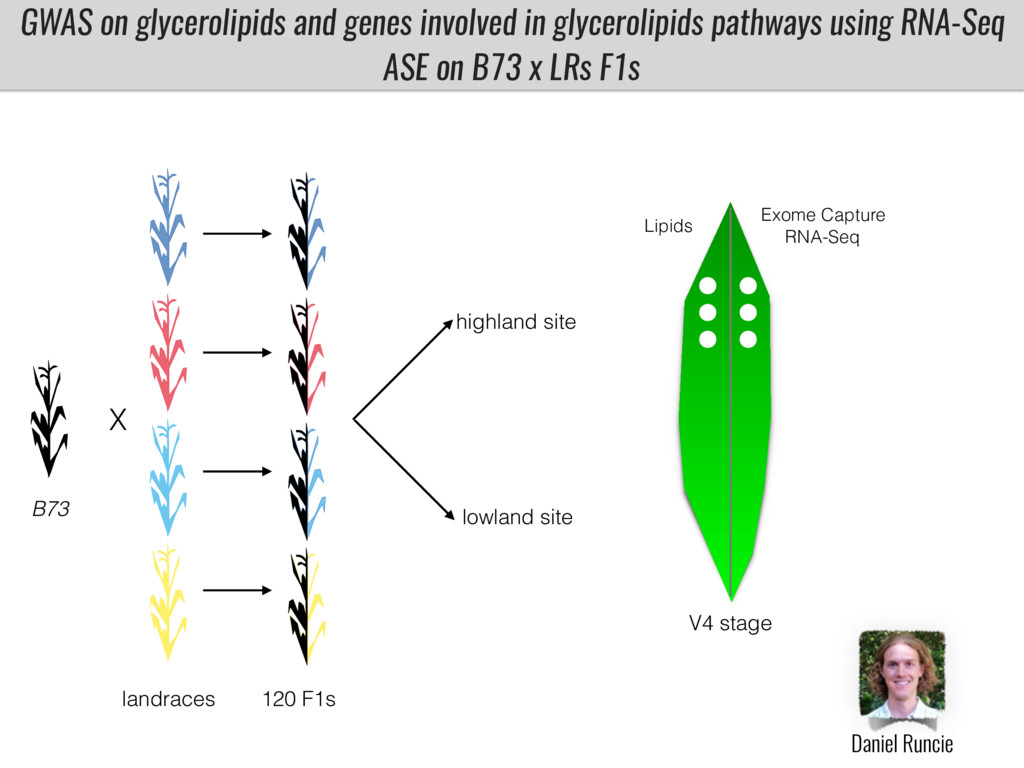
X Daniel Runcie highland site lowland site V4 stage Exome
Capture RNA-Seq Lipids B73 GWAS on glycerolipids and genes involved in glycerolipids pathways using RNA-Seq ASE on B73 x LRs F1s landraces 120 F1s -
Currently working on: -Developing NILs and mutants of candidate genes
to test the possible effect of PT alleles on highland adaptation and under cold/low P conditions. -Identifying possible mutations in the candidate gene that could explain biochemical phenotypes that we observe in B73/PT -Building a Latitudinal Highland Magic Population (High-MAGIC) to analyze the genetic architecture of highland adaptation -Developing markers for candidate gene(s) to explore phenotype-genotypes associations in diversity panels -Identifying divergence of glycerolipids between highland and lowland maize using Qst-Fst. -GWAS on glycerolipids genes involved in glycerolipids pathways using RNA-Seq ASE on B73 x LRs F1s -
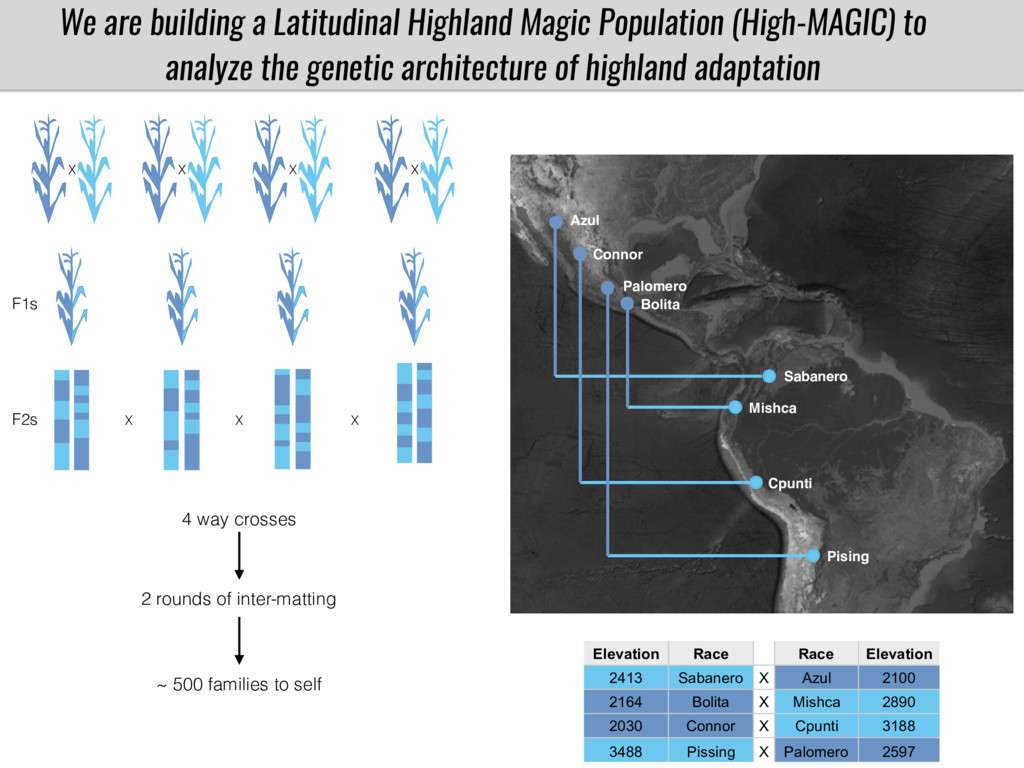
We are building a Latitudinal Highland Magic Population (High-MAGIC) to
analyze the genetic architecture of highland adaptation Azul Connor Palomero Bolita Sabanero Mishca Cpunti Pising Elevation Race Race Elevation 2413 Sabanero X Azul 2100 2164 Bolita X Mishca 2890 2030 Connor X Cpunti 3188 3488 Pissing X Palomero 2597 X F1s X X X F2s X X X 4 way crosses 2 rounds of inter-matting ~ 500 families to self -
Currently working on: -Developing NILs and mutants of candidate genes
to test the possible effect of PT alleles on highland adaptation and under cold/low P conditions. -Identifying possible mutations in the candidate gene that could explain biochemical phenotypes that we observe in B73/PT -Building a Latitudinal Highland Magic Population (High-MAGIC) to analyze the genetic architecture of highland adaptation -Developing markers for candidate gene(s) to explore phenotype-genotypes associations in diversity panels -Identifying divergence of glycerolipids between highland and lowland maize using Qst-Fst. -GWAS on glycerolipids genes involved in glycerolipids pathways using RNA-Seq ASE on B73 x LRs F1s -U-Mu reverse genetics to study the effect of candidate genes on glycerolipid metabolism -
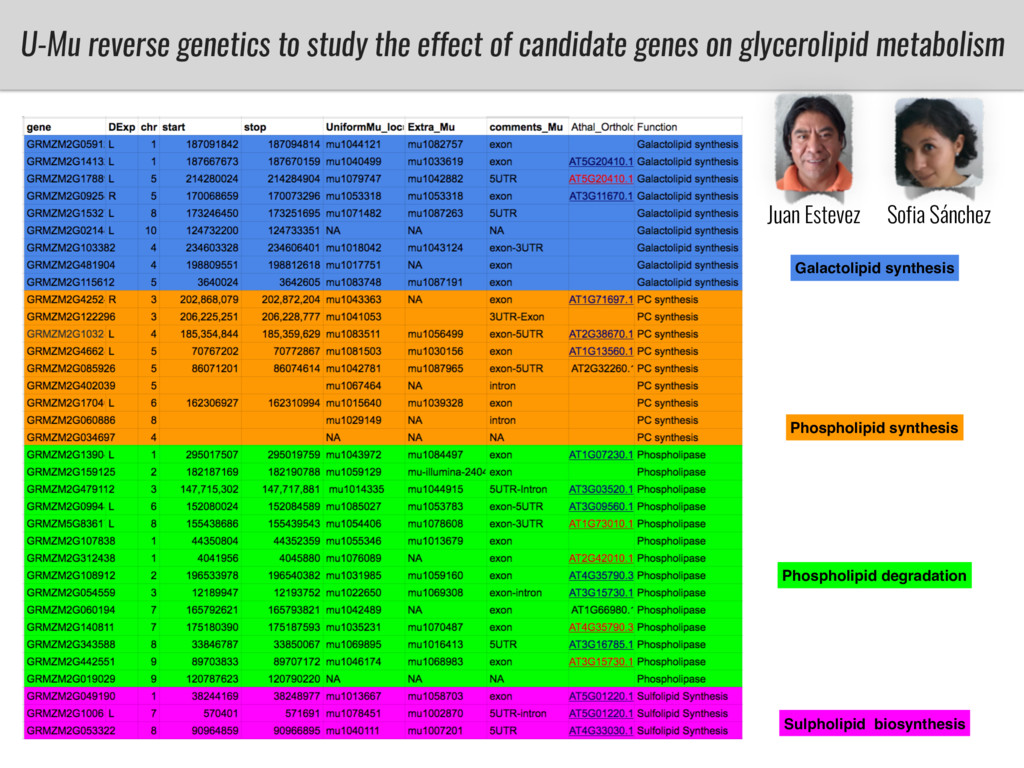
U-Mu reverse genetics to study the effect of candidate genes
on glycerolipid metabolism Galactolipid synthesis Phospholipid synthesis Sulpholipid biosynthesis Phospholipid degradation Sofia Sánchez Juan Estevez -
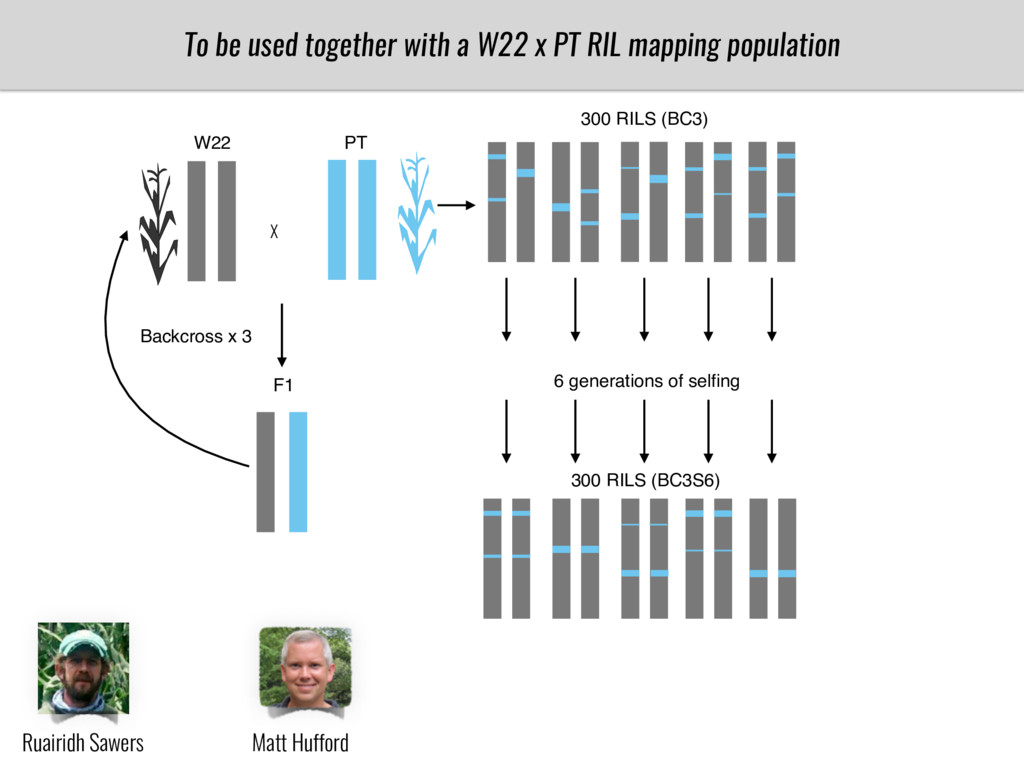
W22 PT X F1 Backcross x 3 300 RILS (BC3S6)
6 generations of selfing 300 RILS (BC3) To be used together with a W22 x PT RIL mapping population Matt Hufford Ruairidh Sawers -
It takes a whole village to grow maize… Karla Juarez
Jeffrey Ross-Ibarra Matt Hufford Daniel Runcie Sherry Flint-García Juan Estevez Ruairidh Sawers Members of the Sawers and Rellan-Álvarez Labs www.highlandadaptation.org Oliver Fiehn Dave Jackson Edgar Demelsa Christoph Benning Kenny Wang Sofia Sánchez Denise Costich -
Allele Specific Expression will allow us to confirm/discover allelic effects
X 40x 40x 80 F1s Daniel Runcie highland site lowland site V4 stage Exome Capture RNA-Seq Lipids B73 Gracias!